GAKI|全球农业知识平台
《世界甘蔗生理生态百科》 / World Encyclopedia of Sugarcane Physiology and Ecology
Phenotypic Plasticity, Acclimation and Genetic Adaptation
Chapter ID: SUG-PHY-V01-C010 | 2026-11-08 | R1 | INDEPENDENT FIRST DRAFT + INITIAL EVIDENCE REVIEW | NOT PUBLISHED
本章研究主问:如何区分短期可逆响应、持续生理驯化、营养繁殖材料的胁迫历史效应,以及群体层面的遗传适应?
Core question: How do short-term reversible responses, sustained acclimation, carry-over through vegetative propagules, and inherited population-level adaptation differ in evidence and mechanism?
证据与权属提醒:本章11篇论文来源的全文、摘要及检索摘录严格分级;未获得的逐株原始数据不得伪造;两幅真实图像沿用既有已核验原件。 出版需待180章全书统一核查。
Evidence and publication note: Eleven original research sources have distinct full-text, abstract or indexed-excerpt scopes. No missing raw observations were imputed. Both authentic images are reused verified assets.
核对维度 / Dimension | 允许的证据 / Appropriate evidence | 不能推断 / Not established |
|---|---|---|
塑性 / Plasticity | 同基因型跨环境 / Within-genotype across conditions | 存在可遗传改变 / Heritable change |
驯化 / Acclimation | 暴露-恢复-再暴露 / Exposure–recovery–rechallenge | 所有阶段均增产 / Universal yield benefit |
延续 / Carry-over | 同来源芽段追踪 / Tracked donor-to-propagule experiment | 跨多代遗传固定 / Stable genetic inheritance |
适应 / Adaptation | 种质谱系+遗传选择 / Heritable population selection | 候选基因即可解释产量 / Candidate gene alone proves yield |
一、研究对象与概念分界 / Scope and conceptual boundaries
1.1 一种基因型并非只有一种表型 / One genotype, multiple phenotypes
甘蔗同一无性系在不同水分、光照、温度和土壤环境中,可形成不同的叶面积、根冠比例、气孔行为、分蘖组成和茎秆糖浓度。 这些差异并不自动表示发生了遗传改变。 严格的表型可塑性是给定遗传材料在不同环境下形成不同表型的能力;一个单点观测不能测量这种能力,必须让同一基因型跨多个环境比较。 可塑性既可能是有利的调节,也可能是资源受限造成的被动衰退。 即使干旱使叶面积明显下降,也不能仅凭变化幅度称其“适应性强”。 [S01][S03]
The same sugarcane clone can differ in leaf area, root-to-shoot allocation, stomatal behaviour, tiller survival and stalk composition across water, light, thermal and soil environments. Such differences do not establish genetic change. Phenotypic plasticity is the capacity of a defined genotype to produce different phenotypes in different environments; a single field observation cannot quantify it. The same clone must be sampled across a meaningful environmental contrast. A large response may be beneficial regulation or merely damage imposed by resource shortage. Severe leaf-area loss under drought, for instance, is not automatically evidence of adaptive plasticity. [S01][S03]
1.2 适应、驯化、逆境记忆与驯化育种 / Adaptation, acclimation, memory and crop domestication
“驯化”在本章需拆分两义:生理驯化(acclimation)是个体在暴露后改变功能状态,可有可逆或跨一段时间持续的部分;作物驯化(domestication)则是人类长期选育导致群体等位基因组成和性状分布改变。 遗传适应通常指种群中可遗传变异经选择发生频率变化。 逆境记忆只是对先前暴露影响后续反应的操作性描述,可能由代谢状态、激素、储藏物、组织结构或表观遗传过程参与,不应在没有机制数据时写成“DNA已经改变”。 [S02][S08][S09]
Two meanings often translated as “acclimation” or “domestication” must remain separate. Physiological acclimation is an exposure-induced change in an individual’s functional state, potentially reversible or persistent over a measurable interval. Crop domestication is historical selection that changes inherited trait distributions and allele frequencies. Genetic adaptation generally refers to heritable population change under selection. Stress memory is an operational term for effects of previous exposure on subsequent responses; metabolism, hormones, reserves, anatomy or epigenetic regulation may contribute. Unless supported by appropriate molecular and inheritance tests, stress memory does not mean that the DNA sequence changed. [S02][S08][S09]
1.3 四个相互独立的研究问题 / Four distinct hypotheses
本章依次检验四个层次:其一,同一无性系的环境反应规范是否显著不同于另一无性系;其二,撤除处理后差异是否恢复或留下持续效应;其三,母本受胁迫是否在营养繁殖芽段的新植株中留下影响;其四,这种差异是否可归因于多代选择形成的可遗传变异。 回答前三问所需的重复暴露与克隆比较,不能替代第四问所要求的遗传及跨代选择证据。 [S01][S02][S07]
Four separately testable questions structure the chapter. First, do clones differ in their reaction norms across environments? Second, does a trait return to baseline after treatment removal or retain a persistent shift? Third, does a prior stress episode in a donor stalk influence a new plant produced from its bud? Fourth, is a difference due to heritable variants shaped by selection across generations? Repeated exposure and clonal comparisons needed for the first three do not substitute for genetic or intergenerational evidence required for the fourth. [S01][S02][S07]
二、结构基础与作用机制 / Structural and mechanistic foundations
2.1 叶片:气孔、光合与水分需求 / Leaves: stomata, photosynthesis and demand
水分不足可降低气孔导度,继而限制二氧化碳进入,但非气孔效应、叶片老化和光化学调节可能同时发生。 两个品种可表现出截然不同的调节路径:一个维持较高气体交换却在强胁迫下下降更剧烈,另一个主要通过减少叶面积降低需水。 叶片瞬时同化高,不保证整个生育期干物质或糖产量高;采样叶龄、叶位、日内时刻和空气水汽压亏缺必须一致。 [S01][S03]
Water shortage may close stomata and restrict CO₂ diffusion, but non-stomatal limitations, leaf ageing and photochemical regulation can also operate. Two cultivars may adopt contrasting strategies: one maintains higher gas exchange under favourable conditions but declines sharply under extreme stress; another restricts demand principally through smaller leaves. High instantaneous assimilation does not guarantee superior lifetime biomass or recoverable sugar yield. Leaf rank, physiological age, measurement time and vapour-pressure deficit must be matched when interpreting gas-exchange data. [S01][S03]
2.2 根系与器官分配 / Roots and allocation across organs
根系深度、表面积、单位根干质量的长度、根系更新速率与根际水势梯度共同决定资源获得机会。 根冠比提高可能来自根生长增加,也可能仅因地上部生长受抑制更大;因此必须同时记录根绝对干质量与地上部干质量。 根窗试验可连续追踪可见根,但根窗接触面不等于整盆三维根系;不同土质和容器大小会影响外推。 [S01]
Root depth, absorbing area, specific root length, turnover and rhizosphere water gradients jointly influence access to resources. An increased root:shoot ratio may arise because roots grew more or because shoots declined faster; absolute root and shoot masses must be reported alongside ratios. Rhizotrons provide valuable longitudinal observations of visible roots but their window surface is not equivalent to a whole three-dimensional root system. Soil texture and container dimensions influence transferability to field crops. [S01]
2.3 先前胁迫对营养繁殖材料的延续 / Carry-over through vegetative propagules
甘蔗靠芽段营养繁殖,芽段不仅携带DNA,也携带储藏物、组织成熟度、芽活力和可能的调节状态。 将来源母株施加三轮干旱处理后,再比较来源于受胁迫与未受胁迫母株的芽段,可以测试“材料历史效应”。 但是若未充分控制芽段大小、节位、养分储备和母株健康状况,就不能将后代差异唯一归因于表观遗传记忆;更不能认定其已构成稳定遗传适应。 [S02]
Sugarcane propagates through buds on stem pieces. A sett transfers DNA but also stored carbohydrates, tissue age, bud vitality and potentially regulatory states. Donor plants exposed to repeated water deficits and then used to generate new plants allow a direct test of origin-history effects. However, without stringent controls on sett size, node position, reserve content and donor health, an offspring difference cannot be assigned uniquely to epigenetic memory. Nor does it demonstrate stable evolutionary adaptation. [S02]
2.4 基因组背景与育种选择 / Genome composition and selection history
现代栽培甘蔗通常为多倍体种间杂交后代,主要承接高糖材料和野生甘蔗的不同基因组贡献。 种间组合与多倍体结构使单个候选基因的表达变化不等同于抗逆表型因果作用。 历史驯化与高糖改良更可能造成多个基因网络、物质分配及开花和分蘖性状的关联选择;2026年大规模基因组研究为选择区域提供线索,但选择扫描不是单基因功能验证。 [S08][S09]
Modern cultivated sugarcane consists largely of highly polyploid interspecific hybrids, drawing contrasting genomic contributions from high-sugar domesticated and wild germplasm. This complexity means an expression shift at a candidate gene is not equivalent to causal proof of stress tolerance. Historical domestication and high-sugar improvement likely involved networks of sugar metabolism, allocation, flowering and tillering traits. A large genomic study published in 2026 identifies candidate selected regions, but a genomic sweep scan is not a functional test of an individual gene. [S08][S09]
三、发育阶段、环境与时间 / Development, environmental context and time
3.1 建苗期与成年蔗的不同可塑性 / Establishment versus established crop
新植蔗早期根系和叶面积尚在形成,短期叶片变化可能迅速影响整株干物质;成年蔗已经具有较大储藏库和较深根系,表现出的缓冲能力、胁迫传递时滞与宿根恢复路径可能不同。 Marchiori等研究持续35天、记录幼龄蔗叶片和根系响应,不应按同一个幅度推断成熟蔗的年产量。 长期田间验证应覆盖新植蔗、第一与后续宿根。 [S01][S07]
Young cane is assembling its root system and leaf area, so short-term trait changes can strongly influence subsequent dry matter. Established stalks possess larger reserves and a more developed root system; buffering, propagation of stress signals and ratoon recovery can differ. The 35-day study of juvenile cane by Marchiori and colleagues describes early growth and cannot be multiplied into a mature-crop annual yield prediction. Longitudinal field validation should include plant cane and several ratoon cycles. [S01][S07]
3.2 干旱强度并非一种通用数值 / Drought intensity is not a universal threshold
土壤基质势(kPa)、土壤相对可用水、叶水势(MPa)与营养液渗透势是四种不同量,不能横向复制一个阈值。 原始根窗实验将水分处理分为高、中、低等级,末期中度处理部分深度约−65至−90 kPa,低水处理曾达到更低值;这些是该实验容器和土壤条件下的观测,而不是全球甘蔗抗旱分级法。 [S01][S02]
Soil matric potential (kPa), fraction of available soil water, leaf water potential (MPa) and solution osmotic potential describe different dimensions. One reported threshold must not be copied between them. The rhizotron experiment partitioned water treatments into high, intermediate and low regimes; the intermediate treatment approached approximately −65 to −90 kPa at the end at a measured depth, while the lowest regime became much drier. These are observed experimental conditions in a particular soil and vessel, not a global classification of sugarcane drought tolerance. [S01][S02]
3.3 胁迫—恢复—再胁迫的完整时间轴 / Stress–recovery–rechallenge chronology
可塑性研究必须记录每次胁迫的开始、强度、结束和恢复时点。 反复轻度干旱后功能有所改善,可能是驯化,也可能来自结构改变或已存活个体的选择偏差。 Marcos等的来源母株接受三次九天干旱,轮次之间复水六天;芽段长成新株后又施加九天渗透胁迫,再复水五天。 只有把两代植株的时间轴拆开,才能明确持续效应来自何处。 [S02]
Plasticity experiments require dates and intensities for each onset, treatment termination and recovery assay. Improved function after repeated mild deficit may reflect acclimation, structural change or survivorship bias. In Marcos and colleagues’ experiment, donor plants experienced three nine-day withholding cycles separated by six days of watering. New propagules were later exposed to a separate nine-day osmotic treatment followed by five days of recovery. Donor and propagule chronologies must be recorded separately before the persistence of any effect can be interpreted. [S02]
3.4 水分历史与管理条件的交互 / Interaction between history and management
预处理可能改变叶片面积、根系配置、抗氧化代谢和初始储藏物,因此相同的第二次处理并不意味着两组植株获得了相同的有效胁迫剂量。 对比应记录净光合、叶水势与实际水耗,而不只记录“停水天数”。 叶片恢复后,干物质亏损未必立即弥补。 长期农艺效果必须同时评价建苗存活率、后续生长和糖产量,而不把重复胁迫推荐为未经验证的田间技术。 [S01][S02]
Pretreatment may alter leaf area, root distribution, antioxidants and initial reserves, so identical second treatments do not necessarily impose identical physiological doses. Comparing groups requires gas exchange, plant water status and actual water use—not merely days since watering stopped. Even if a leaf recovers function, the biomass deficit may persist. Any agronomic claim about deliberate stress conditioning needs field evidence for establishment, later growth and sugar yield; repeated stress is not recommended as a proven management treatment by the experiments reviewed here. [S01][S02]
四、品种、生态区与遗传背景 / Genotypes, regions and genetic background
4.1 品种反应规范与交叉排序 / Reaction norms and rank changes
品种间表现差异至少包含稳定的遗传主效应、环境主效应及基因型×环境互作。 两个品种在充足水分下的排序可能与严重干旱下相反;即使没有排序反转,反应斜率不同也意味着塑性差异。 对“耐旱性”不能只依据单一时期的气孔导度或单株鲜重。 以相同品种跨梯度的性状曲线比较,才可区分高基线表现与强环境响应。 [S01][S03][S07]
Genotypic differences combine genotype effects, environment effects and genotype × environment interaction. Cultivar rankings under ample water may reverse under severe shortage; even without a crossover, different slopes indicate different plastic responses. A cultivar’s drought tolerance cannot be inferred from conductance or fresh mass at one date. Trait reaction norms estimated across a controlled gradient distinguish baseline performance from responsiveness. [S01][S03][S07]
4.2 野生资源不等于现成商业品种 / Wild germplasm is not a ready-to-release cultivar
野生甘蔗材料具有遗传和生态差异,某些材料在光合、抗病、宿根或低投入条件下表现出可利用性状,但并不必然具有高可回收糖产量。 日本琉球地区的比较研究在特定光照和温度下发现部分野生材料的叶片气体交换优于对照栽培品种,这只能支持其候选亲本价值;需要在复杂遗传背景中检验连锁负担、开花和成熟差异,并经多地点田间试验确认育种价值。 [S05][S08]
Wild Saccharum carries genetic and ecological diversity and may contain useful traits for photosynthesis, disease defence, ratooning or low-input performance, yet this does not make a wild accession a high-sugar commercial cultivar. A Ryukyu-region comparison found that particular S. spontaneum lines exhibited higher gas exchange than some cultivated checks under specific light and temperature conditions. Such evidence nominates germplasm for breeding, but linkage drag, phenology, maturity and yield must still be evaluated after crossing and across field environments. [S05][S08]
4.3 多地点与多蔗作周期的适应性 / Multi-location and multi-cycle adaptation
佛罗里达试验在五个地点、三代蔗作周期测试13个候选克隆及3个对照,并设六次田间重复,结果显示地点和品种互作以及不同优势地点群。 该证据是多环境农艺表现,不是对光合酶或膜蛋白机制的直接证明。 单个高产地点可能具有特殊的土壤水位和管理背景,必须记录具体田间处理才能解释互作来源。 [S07]
A Florida study compared 13 experimental clones with three checks at five sites over plant cane, first ratoon and second ratoon, using six field replicates at each site. It found site-dependent performance and distinct groups of favourable environments. These are agronomic genotype-by-environment outcomes, not direct proof of a particular leaf enzyme or membrane transporter mechanism. Site-specific water tables, soils and management need documenting before the physiological source of the interaction can be established. [S07]
4.4 当代基因组扫描的证据位置 / What population genomics does and does not show
甘蔗复杂基因组有利于追踪驯化和改良过程中等位基因来源,但群体分化可能来自选择、种群史、倍性和抽样结构。 2026年一项研究汇总981份甘蔗材料,归入野生、高糖祖先材料及杂交品种群;其扫荡区域和候选基因支持“可能受选择的通路”,不能直接推断每个现代栽培品种均具有同样逆境耐性,更不能把基因型数直接当作独立的田间抗性试验数。 [S09]
Complex sugarcane genomes permit reconstruction of ancestral contributions and candidate regions affected by domestication, but population differentiation may reflect selection, demographic history, ploidy and sampling. A 2026 study analysed 981 Saccharum accessions spanning wild, high-sugar domesticated and hybrid material. Selective regions and genes identify plausible pathways, not universal stress performance of every modern cultivar. The number of resequenced samples must never be counted as an equal number of independent field-tolerance experiments. [S09]
五、原始研究、对立结果与因果链 / Primary experiments, disagreement and inference
5.1 2017巴西根窗实验的主要发现 / Brazilian rhizotron study, 2017
对IACSP95-5000与IACSP94-2094进行2品种×3水分的完全随机盆栽研究,每个组合有三株独立植株,另在同株上多时次测叶片生理。 前者在良好水分下光合能力较高、部分生理参数的塑性更明显,但极端低水情况下其同化可大幅下降;后者在形态指标上塑性更明显,而该幅度并不自动带来更高的干物质积累。 论文的n=15图形点数由3株×5次测量构成,不等于15株生物重复。 [S01]
A factorial greenhouse rhizotron experiment compared IACSP95-5000 and IACSP94-2094 at three water regimes, with three independently grown plants per genotype–water combination. Leaf physiology was repeatedly measured. The former showed higher favourable-water photosynthesis and greater plasticity in several physiological traits, but very low water produced a sharp decline; the latter displayed more morphological plasticity without an automatic biomass advantage. Figures reporting n = 15 represent three plants measured on five dates, not 15 independently randomized biological replicates. [S01]
5.2 2018营养繁殖胁迫历史实验 / Vegetative propagation history experiment, 2018
对IACSP94-2094母株的三轮干旱处理降低了母株叶、茎和根的部分生物量;但其芽段萌芽率在报告中约为95%,高于未受胁迫母株芽段约74%。 来自受胁迫母株的新植株再次受胁迫后,叶片净同化恢复较快。 该结果支持“来源材料历史相关的持续功能差异”,但不意味着母株在每一方面都受益,也不足以证明芽段存在可遗传的DNA序列变化。 [S02]
Three drought cycles imposed on donor cultivar IACSP94-2094 reduced aspects of donor leaf, stalk and root biomass. Yet reported bud sprouting from stressed donors was approximately 95%, compared with approximately 74% from watered donors. Descendant propagules from stressed donors also recovered leaf CO₂ assimilation more rapidly after a later stress. These results support a persistent material-origin effect, not the claim that the donor benefited in every respect, nor evidence that the bud acquired heritable DNA sequence mutations. [S02]
5.3 反例一:形态响应很大但无生长优势 / Counterexample: large morphological change without advantage
若把“可塑性”只解释为变量幅度大,IACSP94-2094叶面积和比叶面积的响应会被误判为普遍优于IACSP95-5000。 然而实际干物质比较并不支持这种简单排序。 合理解释是某些形态变化可能降低消耗,另一些则压缩碳获得;究竟有利于什么目标必须与叶片存活、根生长、水耗和最后产量共同检验。 [S01]
If plasticity is interpreted solely as the size of change, the stronger leaf-area or specific-leaf-area response of IACSP94-2094 would misleadingly be called universally superior. Dry-matter outcomes do not support such a ranking. Some morphological adjustments may save resources whereas others curtail carbon capture. Their value depends on leaf survival, root access, water consumption and ultimately the production target, not the size of a plasticity index alone. [S01]
5.4 反例二:遗传差异与环境驯化不能相互替代 / Counterexample: genotype versus treatment history
北美材料HoCP93-776与TCP02-4587在温室两水分处理中有不同的光合和水分生理表现,说明同一处理条件下材料间存在差异;然而没有共同环境遗传试验或跨代育种证据时,不能直接证明差异是长期当地适应形成的。 另有2014年研究在两个巴西品种中观察到抗氧化同工酶差异,属于具体候选生化机制证据,而不是整株水分利用和糖产量的最终因果链。 [S03][S04]
Greenhouse experiments with North American genotypes HoCP93-776 and TCP02-4587 found different photosynthetic and hydraulic responses under two watering regimes. That establishes genotype-dependent responses under study conditions, not by itself historical local adaptation, which requires a genetic and temporal comparison. A separate 2014 comparison of two Brazilian cultivars found antioxidant isoenzyme differences: these are candidate biochemical mechanisms rather than a complete causal chain to crop-scale water use and harvested sugar. [S03][S04]
5.5 证据冲突的解释等级 / A hierarchy for resolving disagreement
当“干旱处理后恢复快”与“母株生物量降低”同时出现时,不是文献相互否定,而是观测对象、时间尺度和性能指标不同。 研究整合应先核对材料和处理,再区分显著性、效应量与不确定性,接着评估是否有反复验证和田间收获指标。 对只读到摘要的研究,结论只限定为摘要直接报告的观察;不能自行填入其重复数、处理随机化方式或原始图中的平均值。 [S01][S02][S04][S07]
A faster post-drought recovery in progeny and reduced donor biomass are not contradictions: they concern different organisms, periods and outcomes. Evidence synthesis first matches material and treatment, then separates statistical significance, effect size and uncertainty, and finally examines replication and field endpoints. For studies accessible only as abstracts, claims are restricted to observations stated there; replicate counts, allocation procedures and values in inaccessible figures remain unknown rather than being invented. [S01][S02][S04][S07]
原始研究对照矩阵 / Primary evidence comparison matrix
研究 / Study | 材料与实验 / Material and design | 成立与不成立 / Supported & not supported |
|---|---|---|
[S01] Brazil 2017 | 2 cvs × 3 water levels; n=3 plants/cell, repeated leaves | Early plasticity; not 15 independent plants |
[S02] Brazil 2018 | donor 3×9 d drought; 4 blocks progeny | Carry-over; not proof of genome inheritance |
[S03] USA/Brazil 2013 | 2 cvs × 2 water; 4 pots/cell | Cultivar response; not local evolutionary adaptation |
[S07] Florida 2020 | 5 sites × 3 crop cycles × 16 genotypes | G×E in yield; not mechanistic gene evidence |
六、测量方法、数据结构与试验设计 / Measurements, data fields and experimental design
6.1 反应规范和塑性指标 / Reaction norms and plasticity indices
建议以性状y为纵轴、实测环境梯度e为横轴绘制每个品种的反应规范,模型中同时包含品种、环境及其交互项,并报告置信区间。 相对距离塑性指数RDPI可总结跨环境相对变化,但其数学定义依赖性状取值范围;当变量可为负数或接近零时需重新检查稳定性和可解释性。 绝不能把同一植株在五个日期的五次测量当作五个独立随机分配个体。 [S01]
Plot trait y against an observed environmental gradient e for each genotype and fit genotype, environment and their interaction, with uncertainty intervals. The relative distance plasticity index (RDPI) can summarize relative distances across environments, but its definition depends on trait value ranges; variables near zero or taking negative values need particular scrutiny. Five measurement dates on the same plant remain repeated measures of that plant, not five independently randomized experimental units. [S01]
6.2 分层实验单位与混合模型 / Nested units and mixed-effects analysis
设计至少分五层:随机化的地块或容器、植株、分蘖、叶片/节间、叶片重复读数。 每一层记录实际n和取样日期。 对于重复测量,使用植株或小区随机效应、时间自相关和必要的品种×环境×时间固定效应;多个叶片读数不应直接扩大生物重复数。 多地点试验再增加地点、年份、蔗作周期与地块区组,跨点差异需独立估计。 [S01][S02][S07]
At minimum, distinguish randomized plot or vessel, plant, tiller, leaf or internode, and instrumental reread. Record actual sample counts at each level and dates of observation. Repeated-measures models should account for plant/plot random effects, temporal dependence and relevant genotype × environment × time terms; multiple leaf readings cannot inflate the number of biological replicates. Multi-site studies add site, season, ratoon cycle and block effects, with uncertainty of cross-location contrasts estimated explicitly. [S01][S02][S07]
6.3 水分与光合测量的口径 / Water and gas-exchange measurements
气孔导度gₛ、同化速率A、蒸腾E、水分利用效率A/E及内在效率A/gₛ应分别登记单位、仪器气室设置、CO₂浓度、光合光子通量、叶温和采样时间。 不同分母的“水分利用效率”不应互换。 气室测得的瞬时WUE不代表整个生长周期的蒸散效率。 相对含水量RWC必须保存鲜质量、复水饱和质量、干质量的采样流程与计算基准。 [S01][S02][S03][S06]
Record stomatal conductance gₛ, assimilation A, transpiration E, instantaneous A/E and intrinsic A/gₛ with units, chamber CO₂, photon flux, leaf temperature and sampling hour. These efficiencies use distinct denominators and are not interchangeable. Instantaneous chamber WUE is not equivalent to seasonal evapotranspiration efficiency. Relative water content requires the fresh, rehydrated-turgid and dry mass protocol to be stored along with the formula and tissue basis. [S01][S02][S03][S06]
6.4 种源、克隆谱系与可追溯性 / Propagule lineage and reproducibility
每根芽段应有唯一材料ID,并记录母株编号、母株历史处理、剪取日期、芽段长度、节位、芽龄、芽活性、预处理、培养条件及种植后时间。 若母株多个芽段进入同一组,应保留母株来源为潜在聚类层,防止把同一来源的全部芽段当作彼此独立。 若声称表观遗传传递,应添加DNA甲基化或染色质证据,并设计无胁迫传代排除短期储藏物效应。 [S02]
Assign each sett a unique ID and record donor identity and treatment history, cutting date, length, node, bud developmental stage, viability, pretreatment, culture conditions and planting age. Multiple propagules from one donor require donor identity as a possible clustering level; they are not necessarily fully independent biological histories. Claims of epigenetic transmission require relevant methylation or chromatin measurements and unstressed propagation cycles capable of separating persistent regulation from temporary reserve effects. [S02]
6.5 实际数据库字段与质量控制 / Operational database schema and QC
结构化系统应提供源论文DOI、原文位置、访问层级、试验材料、环境坐标、栽培周期、随机化单位、观测单位、处理时间线、原始观察/发表汇总/设计参数分类、分析方法、主张范围、反证与图像SHA-256。 对于从摘要获取的数值,不得标记为全文已核验。 不同论文如重用同一试验材料或数据集,应保留共享实验ID,不重复累计独立验证次数。 空缺值使用null并说明原因。 [S01][S02][S07]
The evidence system must capture DOI, article locator and access level, study material, environmental context, crop cycle, randomized and observed units, complete treatment chronology, numeric evidence type (raw observation, published summary or design parameter), analysis, claim scope, contradicting evidence and image SHA-256. Numbers visible only in abstracts cannot be certified as full-text-verified. Publications sharing a trial or dataset require a shared experiment identifier, not separate counts of independent validation. Unknown values remain null with a reason. [S01][S02][S07]
结构化数据必要字段 / Required database fields
字段 / Field | 取值及数据质量要求 / Required content |
|---|---|
genotype_id / clone_lineage | 物种、品种、谱系和母株关联ID / taxon, cultivar and donor lineage |
environment_exposure | soil Ψm; leaf Ψ; atmospheric VPD; dates; leaf rank; growth stage |
independent_unit / repeated_n | 地块/容器/植株/叶片/重测分层 / nested units and repeated sampling |
numeric_record_type | design / published_summary / raw_observation / digitized / derived |
claim_scope / limitations | 材料、地点、时刻、因果级别与待核项 / restricted inference |
media_rights / sha256 | 来源原件、作者、许可、尺度及内容哈希 / authenticity and license |
七、真实图像、照片用途与图注 / Authentic images and evidence use
7.1 田间实景的作用与边界 / Field photographs as context, not a treatment contrast
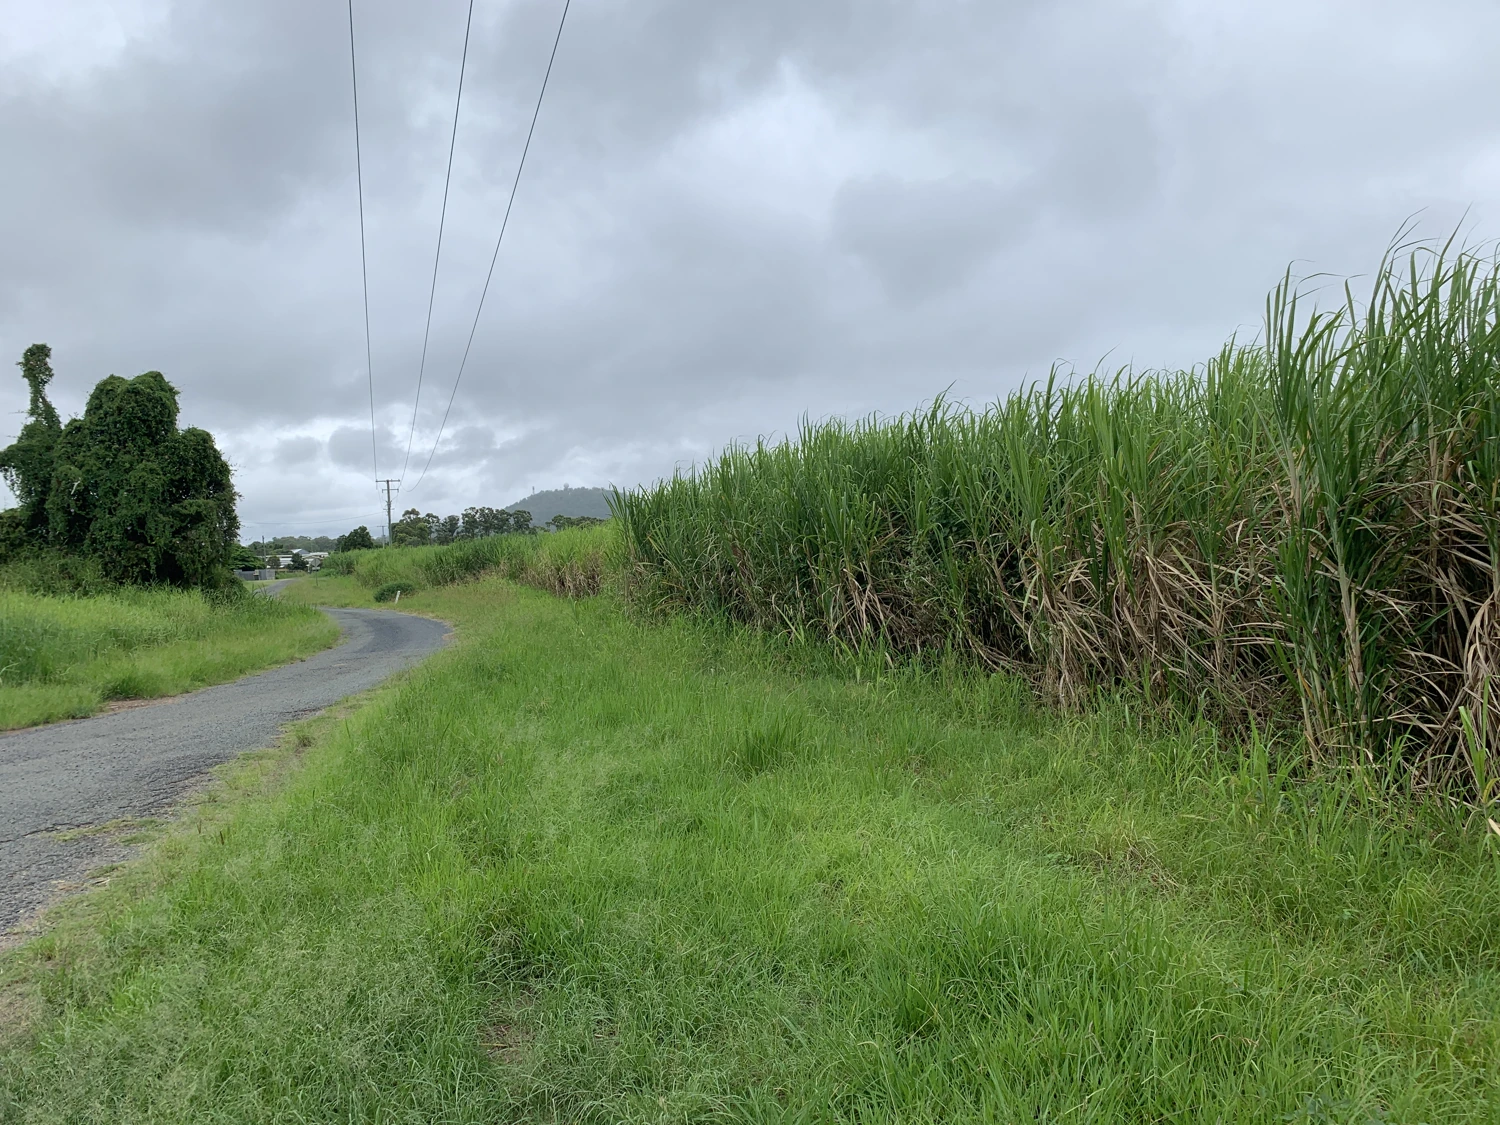
本章复用一幅有作者与许可的澳大利亚甘蔗田原始实景照片,用于说明成熟群体、冠层和田间环境,不据此推测品种、处理、水分状况或产量。 摄影照片本身不是对照试验,同一张照片无法证明遗传适应或可塑性。 未来若取得同一品种、同视角、同成像条件的跨环境原图,应同时记录种植设计和拍摄日期,才能用于叶面积/冠层结构的定量比较。
The chapter reuses an attributed and licensed field photograph from Australia to document a mature canopy and real cropping context. It is not used to infer cultivar identity, irrigation treatment, measured water status or yield. A single photograph is not a controlled comparison and cannot establish genetic adaptation or plasticity. For future paired field images, genotype, camera position, illumination, dates and randomized field design must accompany the files before quantitative comparisons are attempted.
7.2 显微图片的证据类型 / What anatomical micrographs can substantiate
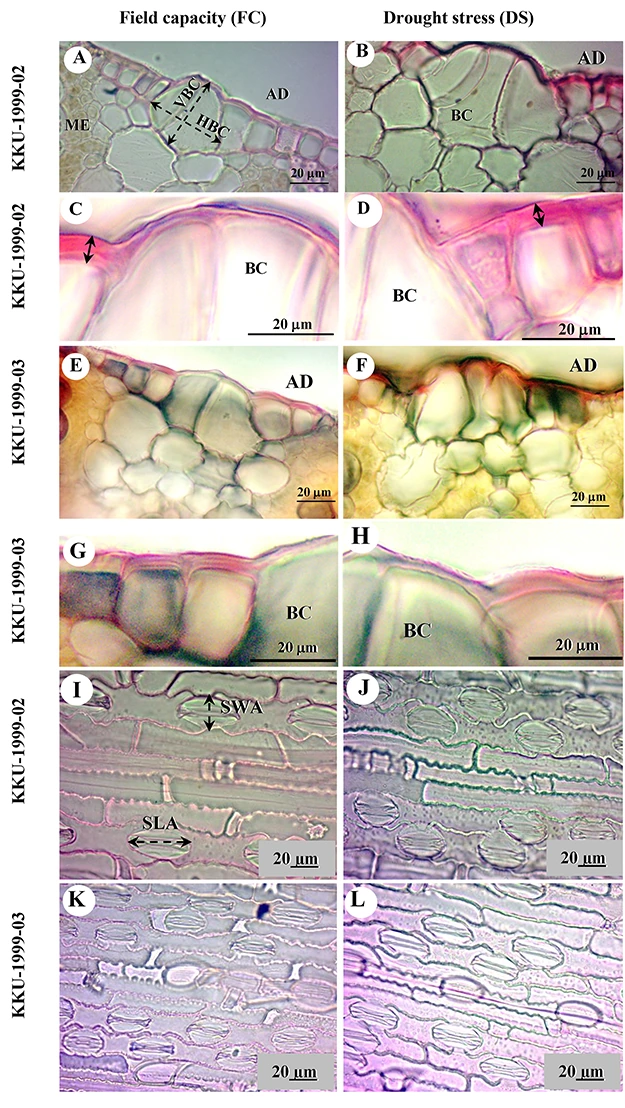
本章另复用甘蔗叶片气孔及组织显微图版,展示真实解剖性状及水分条件下的组织对照。 比例尺与面板代号来自原发表研究;不同面板不能当作多篇独立研究。 显微差异可以启发“表型由结构与功能共同决定”的假说,但需配合同批次生理测量和统计才足以解释功能性能。 图像许可、原作者与SHA-256继续沿用已核验主资产记录。
An existing licensed sugarcane epidermal micrograph plate shows authentic anatomy and panels collected under contrasting water conditions. Scale bars and panel identifiers derive from the original publication; multiple panels from one paper do not constitute independent studies. Anatomical differences can motivate hypotheses linking structure with performance, but paired gas-exchange measurements and appropriate replication are needed for functional inference. Original authorship, licence and SHA-256 remain attached to the verified source asset.
7.3 未取得原图的缺口 / Unacquired figures stay pending
另检索到美国农业部历史甘蔗田照片(Scott Bauer,1997年12月,佛罗里达);来源页标注为美国联邦政府公务作品公有领域,但本章原件下载失败,故只保留“线索、许可信息、失败状态”,不在本章嵌入也不记为新增取得图片。 后续可替换为另外一张合法的新图,而不对此同一原件反复尝试。
A historical USDA image credited to Scott Bauer (Florida, December 1997) was found with a public-domain federal-work statement. The original file download failed in the source review. It therefore remains a documented lead, not an embedded or newly acquired asset. A distinct licensed photograph may be sought in a later evidence round without repeated attempts on this failed file.
网页预览经过缩放或格式转换,未裁切;原比例尺与标签保留。 / Web preview resized or re-encoded without cropping; original scales and labels retained.
图10-1 澳大利亚真实甘蔗田外观,展示成熟群体与田间环境;该图不能证明品种差异或逆境效果。 摄影:Kerry Raymond,2022年,CC BY 4.0。
Fig. 10-1. Authentic Australian sugarcane field context; the image does not demonstrate cultivar differences or stress effects. Photograph: Kerry Raymond, 2022, CC BY 4.0.
网页预览经过缩放或格式转换,未裁切;原比例尺与标签保留。 / Web preview resized or re-encoded without cropping; original scales and labels retained.
图10-2 甘蔗叶表皮显微图版(原论文多面板及20 μm比例尺)。 此类原始解剖图可观察组织性状,但不能单凭图像建立耐旱因果关系。 原研究作者,CC BY 4.0。
Fig. 10-2. Original sugarcane epidermal micrographs with panel labels and 20-µm scale bars. Anatomy alone does not prove drought-tolerance causality. Original research authors, CC BY 4.0.
图版原件与权属记录采用资产ID:SUG-PHY-C001-IMG-002 / SUG-PHY-C001-IMG-003;本章没有新增取得这两张图片。
八、适用边界、研究缺口与结论 / Transferability, gaps and conclusions
8.1 三个结论不应混写 / Three conclusions must not be merged
第一,同一遗传材料面对水分变化可以产生多个表型;第二,先前处理可使芽段来源的新植株表现不同;第三,长期选择改变甘蔗种质的可遗传组成。 三者涉及不同的材料、时间尺度和因果证据。 将短期生理恢复称为“基因驯化成功”,将选择扫描称为“田间耐旱率已提高”,都超过了证据。 对甘蔗品种实用性评价必须另行测定生长稳定性、蔗糖产量和机械收获适宜性。 [S01][S02][S08][S09]
Three propositions have different subjects, time scales and causal requirements: a fixed genotype produces different phenotypes across environments; a donor’s treatment history alters subsequent propagule performance; and long-term selection changes inherited germplasm composition. Better short-term recovery cannot be called successful genetic domestication, and a sweep scan does not establish improved field survival or drought yield. Practical cultivar evaluation still requires crop stability, recoverable sucrose production and compatibility with commercial field operations. [S01][S02][S08][S09]
8.2 需要补足的实验 / Priority experiments
推荐的检验顺序是:基因型×多环境×重复蔗作周期试验;统一水势与叶位的时间序列;复水后长时间干物质补偿;以同母株多芽段追踪延续效应;无胁迫条件下营养繁殖后连续两代检验持续性;最后将遗传标记与功能、收获和抗逆成本相联系。 优先公开逐小区、逐株原始数据与随机化代码,并同步保存真实图像原件。 当前可检索研究未满足全部条件,因此不能发布适用于所有国家的阈值或商品化胁迫预处理规程。
Priority work comprises genotype × multi-environment × ratoon-cycle trials; time series standardized by water status and leaf rank; long-term biomass catch-up after rewatering; tracking multiple setts from identified donors; testing carry-over across successive unstressed vegetative generations; and finally linking genetic markers to function, yield and tolerance costs. Plot-level and plant-level observations, randomization records and original images should be shared where lawful. The reviewed studies do not jointly meet these requirements, so no global drought threshold or commercial preconditioning protocol is recommended.
8.3 本章科研结语 / Scientific synthesis
本章建立的核心观点不是“越可塑越好”,而是“必须说明哪项表型、在什么环境梯度、什么生育阶段、以什么成本改善了哪一种结果”。 原始研究已证实甘蔗幼株水分响应具有基因型差异,营养繁殖材料的先前胁迫历史可产生持续后效,野生及栽培材料间存在可供育种的遗传多样性;不过,机制、长期收益和多地点生产力之间仍需独立验证。
The central conclusion is not “more plasticity is better” but “which phenotype, under what gradient and developmental stage, improved which outcome at what cost?” Primary studies demonstrate genotype-dependent water responses in young cane, carry-over effects associated with stress history of vegetative material, and genetic diversity of potential value to breeding. The links from candidate mechanisms to sustained advantage and multi-location sugar productivity, however, demand separate field validation.
双语术语 / Bilingual glossary
中文 / Chinese | English |
|---|---|
表型可塑性 | phenotypic plasticity |
环境反应规范 | reaction norm |
生理驯化 | physiological acclimation |
作物驯化 | crop domestication |
遗传适应 | genetic adaptation |
逆境记忆 | stress memory |
遗传×环境互作 | genotype × environment interaction |
气孔导度 | stomatal conductance |
净同化速率 | net CO₂ assimilation rate |
内在水分利用效率 | intrinsic water-use efficiency |
瞬时水分利用效率 | instantaneous water-use efficiency |
根冠比 | root-to-shoot ratio |
比叶面积 | specific leaf area |
根系比长度 | specific root length |
叶水势 | leaf water potential |
相对含水量 | relative water content |
母株历史 | donor-plant history |
营养繁殖芽段 | vegetative propagule / sett |
干旱预处理 | drought preconditioning |
再胁迫 | stress rechallenge |
恢复速率 | recovery rate |
可逆性 | reversibility |
选择扫荡 | selective sweep |
多倍体 | polyploidy |
独立试验单位 | independent experimental unit |
生物重复 | biological replicate |
技术重复 | technical replicate |
重复测量 | repeated measure |
相对距离塑性指数 | relative distance plasticity index |
反证 | contradictory evidence |
抗逆代价 | cost of stress tolerance |
分层混合模型 | hierarchical mixed model |
候选基因 | candidate gene |
物候阶段 | phenological stage |
原始研究与来源范围 / Original sources and access scope
[S01] Marchiori et al. (2017) Physiological Plasticity Is Important for Maintaining Sugarcane Growth under Water Deficit. DOI: 10.3389/fpls.2017.02148.
Source URL: https://www.frontiersin.org/journals/plant-science/articles/10.3389/fpls.2017.02148/full | access: FULL_HTML_READ
[S02] Marcos et al. (2018) Drought tolerance of sugarcane propagules is improved when origin material faces water deficit. DOI: 10.1371/journal.pone.0206716.
Source URL: https://pmc.ncbi.nlm.nih.gov/articles/PMC6306257/ | access: FULL_HTML_READ
[S03] Silva et al. (2013) Photosynthetic capacity and water use efficiency in sugarcane genotypes subject to water deficit during early growth phase. DOI: 10.1590/S1516-89132013000500004.
Source URL: https://www.scielo.br/j/babt/a/jzBcSWs3K7jHj67wKXpQxNn/?lang=en | access: FULL_HTML_READ
[S04] Boaretto et al. (2014) Water stress reveals differential antioxidant responses of tolerant and non-tolerant sugarcane genotypes. DOI: 10.1016/j.plaphy.2013.11.016.
Source URL: https://pubmed.ncbi.nlm.nih.gov/24308986/ | access: ABSTRACT_READ
[S05] Nose et al. (1994) Variations in Leaf Gas Exchange Traits of Saccharum Including Feral Sugarcane, Saccharum spontaneum L.. DOI: 10.1626/jcs.63.489.
Source URL: https://www.jstage.jst.go.jp/article/jcs1927/63/3/63_3_489/_article/-char/en | access: ABSTRACT_READ
[S06] Genetic variation transpiration study (2016) Genetic variation in transpiration efficiency and relationships between whole plant and leaf gas exchange measurements in Saccharum spp. and related germplasm. DOI: 10.1093/jxb/erv505.
Source URL: https://academic.oup.com/jxb/article/67/3/861/2893264 | access: ABSTRACT_READ
[S07] Florida multi-environment group (2020) Genotype-by-environment interaction analysis across three crop cycles in sugarcane. DOI: 10.1080/15427528.2020.1817220.
Source URL: https://www.tandfonline.com/doi/full/10.1080/15427528.2020.1817220 | access: ABSTRACT_READ_FULL_BLOCKED
[S08] Zhang et al. (2018) Allele-defined genome of the autopolyploid sugarcane Saccharum spontaneum L.. DOI: 10.1038/s41588-018-0237-2.
Source URL: https://www.nature.com/articles/s41588-018-0237-2 | access: FULL_TEXT_EXCERPT_FROM_SEARCH
[S09] Sugarcane genome architecture team (2026) Genetic architecture of sugarcane traits in a polyploid genomics framework. DOI: 10.1038/s41586-026-10576-7.
Source URL: https://www.nature.com/articles/s41586-026-10576-7 | access: SEARCH_EXCERPTS_ONLY
[S10] Khuimphukhieo et al. (2024) Assessing Drought Stress of Sugarcane Cultivars Using Unmanned Vehicle System (UAS)-Based Vegetation Indices and Physiological Parameters. DOI: 10.3390/rs16081433.
Source URL: https://www.mdpi.com/2072-4292/16/8/1433 | access: ABSTRACT_READ_FULL_429
[S11] Lunn et al. (2024) Greater aperture counteracts effects of reduced stomatal density on water conductance in sugarcane. DOI: 10.1093/jxb/erae271.
Source URL: https://digitalcommons.unl.edu/agronomyfacpub/1777/ | access: ABSTRACT_READ
编写状态与下一章 / Editorial status and next chapter
第010章:初稿完成;首轮来源核查完成但仍存在摘要层与全文待核主张;全书级审核、独立复现实验审核及出版审核未完成。 002—009离线正文不应被当作Library主目录中已登记文件。
Chapter 010: draft completed; initial source review performed, with remaining abstract-only claims. Whole-book review, independent replication assessment and publishing approval are still pending.