《世界甘蔗生理生态百科》 / World Encyclopedia of Sugarcane Physiology and Ecology
Environmental Factors and Limiting Processes
Chapter ID: SUG-PHY-V01-C009 | R1 research draft / 研究初稿 | 2026-11-08 | NOT PUBLISHED / 尚未发布
本章主问:怎样判断观测到的生长限制来自哪种环境因子及其作用环节?
Guiding question: Which environmental factors and physiological steps cause the observed limitation of crop growth?
写作边界:所有结论均限定材料、生态区、试验单位、时间与测量尺度;未取得的原始观测数据不补造。 全文中[S01]—[S13]对应文末的可核对来源。
Evidence status: 13 indexed primary studies, with separate access scopes.
研究层级 / level | 典型变量 / typical variables | 典型错误 / invalid shortcut |
|---|---|---|
环境暴露 / Exposure | PPFD、VPD、叶温、θv、ECe、根区氧 | 用年降水量代替根水势 / Rainfall ≠ root water status |
近端生理 / Proximal physiology | gs、A、叶水势、Fv/Fm、酶活性 | 一项指标代表所有限制 / One marker ≠ whole process |
生长整合 / Growth integration | 叶面积、分蘖、干物质、节间伸长 | 单叶速率代替群体生长 / Leaf rate ≠ crop growth |
经济产量 / Harvest output | 鲜蔗产量、可回收糖率、糖产量 | Brix代替糖产量 / Brix ≠ sugar yield |
一、研究对象、限制的定义与可检验问题 / Research domain, limiting processes and hypotheses
1.1 环境因子并不是生理过程 / Factor is not process
甘蔗生理生态学中的环境因子包括光合有效辐射、冠层光质、叶温与夜温、根区水分、空气水汽压亏缺、根区氧、土壤盐分、养分供给以及相互作用的管理条件。 “缺水”是外部状态,不能直接替代“气孔扩散受限”或“叶片扩展受限”这样的中间机制。 相同的田间减产现象也可能分别源于芽萌发降低、有效茎数减少、单茎干物质积累变慢或茎汁分配改变。 研究必须把外部暴露、器官功能、全株响应和收获结果分层记录,不能把同期相关性写成因果关系。
Environmental exposures include photosynthetically active radiation and light quality, leaf and night temperature, root-zone water supply, atmospheric vapour-pressure deficit, oxygen around roots, salinity, nutrient supply and the management conditions that modify each exposure. “Water shortage” is an environmental state, not a synonym for stomatal limitation or curtailed leaf expansion. The same decline in harvested cane may arise from failed establishment, fewer surviving stalks, reduced stalk dry-matter production, or altered allocation. Exposures, organ-level mechanisms, whole-plant responses and harvest outcomes must therefore be represented as distinct variables rather than collapsed into a single correlation.
1.2 限制因子、限制步骤与共同限制 / Limiting factor, process and co-limitation
若提高某一资源的可利用量能够在其他条件保持足够接近时增加目标过程的速率,则该资源可能构成当前限制因子;但这种实验结论只适用于相应阶段与背景。 即使施水后净同化速率提高,也不一定证明长期茎重受水分单独控制。 多个约束可以同时存在:高温提升蒸发需求、土壤缺水限制根系供给,最终共同改变气孔和叶能量平衡;积水改变根区供氧、根系伸长和营养吸收。 限制步骤会随日内时刻、叶龄、作物龄期与胁迫历史转移。 [S01][S03][S07][S12]
A factor is operationally limiting when a defensible intervention that changes its availability alters the target physiological rate under otherwise comparable conditions. This conclusion is conditional on the stage, genotype and background environment. Recovery of leaf CO₂ assimilation after watering does not by itself prove that final stalk yield is limited solely by water. Constraints can co-occur: heat raises evaporative demand while dry soil restricts supply, jointly altering stomata and leaf energy balance; flooding reduces root-zone aeration and may influence extension and nutrient uptake. The bottleneck can shift with time of day, tissue age, crop phase and stress history. [S01][S03][S07][S12]
1.3 四级因果链与可证伪假说 / A four-level causal chain
本章采用“环境暴露→近端生理指标→生长整合→产量表现”四级证据链。 例如假说H09-A:在土壤含水下降但叶温未明显变化的早期,气孔导度先下降,随后单叶同化速率和绿色叶面积下降,最终地上部干物质降低。 测试需要同时观察土壤水分、叶水势、气孔导度、光合速率和分次生物量;如导度不降而叶面积仍缩小,则必须改写机制。 假说H09-B:短期涨水在成年蔗中未必立即降低净光合,而建苗期长时间积水可抑制生物量,两者并不矛盾。 [S01][S03][S04]
The working chain is exposure → proximal physiology → integrated growth → harvested performance. Hypothesis H09-A predicts that as soil water falls, stomatal conductance may change before leaf carbon assimilation, green leaf area and ultimately shoot mass decline. It must be tested jointly against soil moisture, leaf water potential, conductance, gas exchange and sequential biomass; a contrary pattern requires a revised mechanism. Hypothesis H09-B predicts that brief flooding need not immediately depress leaf assimilation in established cane, whereas longer flooding during establishment may reduce biomass. Both outcomes can be valid within their respective stages. [S01][S03][S04]
二、器官结构与限制步骤 / Organ structures and physiological control points
2.1 叶片:扩散与生化能力 / Leaf: diffusion and biochemical capacity
叶片对光、温度、水势和空气湿度的响应并非一项单独的“光合能力”。 光照决定可利用光子及冠层内的空间分布;气孔调节CO₂供应并影响蒸腾;叶绿体和C4碳浓缩过程则决定生化固定潜能。 低温实验显示,不同甘蔗材料在10°C下的净光合下降程度不同,PPDK与NADP-MDH活性变化与材料差异相伴,但不能因此断定所有受冷甘蔗均以单个酶作为唯一瓶颈。 [S06] 气孔导度也不能被无条件当作抗旱性指标。 [S12]
Leaf photosynthesis cannot be reduced to one parameter called “capacity”. Photon flux and canopy optics determine light availability; stomata regulate CO₂ diffusion and water loss; chloroplast and C4-cycle reactions affect biochemical fixation. A 10°C chamber study found contrasting rates of photosynthetic decline among sugarcane materials, accompanied by different changes in PPDK and NADP-MDH activities, but it does not establish that one enzyme is the sole limiting step for every chilled sugarcane crop. [S06] Likewise, conductance is not a context-free measure of drought tolerance. [S12]
2.2 根系:吸水、供氧和离子稳态 / Roots: water, oxygen and ionic homeostasis
根系在不同胁迫下可能表现为不同限制通路。 干旱首先改变根土界面的水势梯度,盐分同时带来渗透胁迫与潜在离子毒性,积水则影响氧扩散和能量供应。 蔗根和蔗茎组织的形成阶段、通气组织发育以及先前适应历史,决定短期积水能否被缓冲。 美国佛罗里达的渗漏计试验在部分短淹周期观测到中性或正向的单叶气体交换响应;这不能推断长期缺氧也无害。 [S03][S05] 盐处理盆栽中的外加NaCl浓度亦不等于田间土壤电导率。 [S08]
The root compartment has distinct control pathways. Drought changes the water-potential gradient between soil and root, salinity combines an osmotic challenge with potential ion toxicity, and saturation constrains oxygen diffusion and energy metabolism. Root developmental stage, aerenchyma formation and pre-exposure history influence whether transient flooding is buffered. Florida lysimeter experiments reported neutral or sometimes positive single-leaf gas-exchange responses during short flood cycles; these observations cannot be extended to all prolonged oxygen limitation. [S03][S05] Nominal NaCl additions in a pot treatment are not field electrical-conductivity thresholds. [S08]
2.3 茎秆与源库:总量和浓度 / Stalk source–sink: quantity versus concentration
茎秆伸长消耗同化碳并改变库需求,成熟过程中可溶性糖含量可能提高,但糖浓度增加并不等价于单位面积可回收糖产量增加。 热、旱和盐分可以同时改变叶片供碳、节间生长、组织含水量及蔗糖代谢,单次Brix或SPAD值均不是全流程结果。 只有将叶片受光、茎数、节间生长、干物质和质量检测串联,才可能把环境过程与经济产量连接起来。 [S09][S10]
Stalk extension creates sink demand while maturation may increase soluble sugar concentrations; a higher concentration is not automatically a higher recoverable sugar yield per hectare. Heat, water deficit and salt exposure can simultaneously alter carbon supply, internode growth, tissue hydration and sucrose metabolism. A single Brix or SPAD observation is not a full production outcome. Canopy light capture, stalk population, internode development, dry matter and appropriate quality assays must be linked before environmental mechanisms are connected to harvest economics. [S09][S10]
三、发育阶段、时间与暴露历史 / Development, time and exposure history
3.1 早期建苗与快速生长 / Establishment versus grand growth
芽萌发、初生根建立、分蘖形成与快速伸长期受到的约束不同。 Glaz与Lingle的三个盆栽试验针对约9厘米高的初植蔗,水淹0—6周,叶、茎和根生物量随淹水时间增加通常下降;而已建立蔗株的短周期淹水资料却不一定显示即时光合损害。 看似冲突的研究提示,发育阶段和暴露长度应作为一等数据字段,不可在“耐涝/不耐涝”二分标签中丢失。 [S03][S04]
Bud emergence, adventitious-root establishment, tiller recruitment and rapid stalk extension have different constraints. Three pot experiments with recently planted cane of approximately 9 cm starting height found declining leaf, stalk or root biomass with flood duration of 0–6 weeks; studies of established cane under short flooding cycles did not necessarily observe immediate photosynthetic injury. Such apparent disagreement illustrates why crop phase and duration must remain first-class data fields rather than disappear into a binary “flood tolerant” label. [S03][S04]
3.2 日尺度、小时尺度和恢复阶段 / Diurnal timing, acute exposure and recovery
气孔导度可以在分钟量级随光照和水汽压亏缺改变,叶片荧光与光合酶状态可在小时—数日内响应;茎秆生物量和收获产量是长时间积分量。 Du等的10°C处理比较了4、28和52小时,Mathur等的冷处理采用3日暴露及3日恢复,这些尺度与年产量不可混写。 恢复应至少区分回到标准环境后的功能恢复、组织损伤修复和后续生长补偿,而不能只看单次气孔重新开放。 [S06][S11][S13]
Conductance may shift on a minute scale following changing light and vapour demand, while fluorescence and enzyme responses can unfold over hours or days; stalk biomass and harvest yield integrate much longer intervals. Du and colleagues sampled after 4, 28 and 52 h at 10°C, while Mathur and colleagues applied three days of chilling followed by three days of recovery. Those time scales cannot be described as annual productivity effects. Recovery itself must distinguish return of short-term function, tissue repair and later compensatory growth. [S06][S11][S13]
3.3 新植蔗、宿根蔗与季节反转 / Plant cane, ratoon and seasonal reversals
新植蔗与宿根蔗具有不同的初始储藏器官、根系再生速度和群体年龄结构。 环境限制在雨季可能以根区氧限制呈现,旱季则表现为水分供需失衡;同一地块也可能先旱后涝。 佛罗里达2005—2007年试验跨新植蔗、第一宿根和第二宿根,同时比较地下水位与周期淹水,结论依品种、周期及指标而变;因此不能挑选某一作物季作为通用响应。 [S05]
Plant cane and ratoons begin from distinct storage structures, root-renewal trajectories and age distributions. In wet months the putative bottleneck may be root oxygen, whereas in dry months it may be hydraulic supply; the same field can experience both in sequence. A Florida study spanning plant cane, first ratoon and second ratoon across 2005–2007 assessed water-table depth and periodic flooding, finding outcomes dependent on cultivar, cycle and measured variable. A single crop season should therefore not be marketed as a universal response. [S05]
四、环境梯度与机制判别 / Environmental gradients and mechanism discrimination
4.1 辐射与遮阴:叶片响应不等于群体响应 / Light and shade
弱光限制光合电子传递和碳同化,但叶片光响应曲线的饱和点不等于冠层最优叶面积指数。 田间六个高糖品种的光响应拟合显示,部分材料在偏热湿条件下出现强光抑制,GT02-467在该试验中未呈现相同模式;模型选择也影响参数估计。 [S10] 因此必须同时保存PPFD、叶位、叶温、测量时刻、饱和前后光区间和光曲线拟合式。 不能据单叶曲线直接推荐全国通用的密植制度。
Low irradiance restricts electron transport and carbon gain, yet the light-saturation point of a leaf is not the optimum canopy leaf-area index. A field comparison of six high-sugar varieties reported high-light inhibition under warm humid conditions for most tested varieties but not GT02-467; fitted parameters also depended on model form. [S10] Preserve PPFD, leaf rank, leaf temperature, time of measurement, pre- versus post-saturation range and the fitted function. A single-leaf curve cannot by itself justify a universal national planting density.
4.2 温度:直接动力学与水分耦合 / Temperature: kinetics and water coupling
低温降低部分C4反应速率、改变气孔与光系统,极端高温可同时损害膜结构与酶体系。 需要区分气温、叶温、昼夜温差、胁迫持续时间及测量温度。 Du等在10°C暴露后再分别于10°C和30°C测光合,强调“受冷历史”和“当下测量温度”不是同一变量。 [S06] Kohila与Gomathi的盆栽试验采用三次重复、15日处理,日/夜高温为45/32±2°C(对照37/28±2°C);在不同材料和阶段观测到叶绿素、气体交换及膜损伤相关指标的差异。 [S09] 所谓单一的“甘蔗最适温度”缺乏充分定义。
Cold conditions can slow C4 reactions and alter stomata and photosystems, whereas extreme heat may impair membranes and enzymes. Air temperature, leaf temperature, night temperature, exposure duration and measurement temperature must be separated. Du and colleagues measured chilled leaves both at 10°C and after transfer to 30°C, explicitly distinguishing exposure history from instantaneous assay temperature. [S06] In a randomized three-replicate pot study, Kohila and Gomathi exposed plants for 15 d to 45/32±2°C (control: 37/28±2°C, day/night), observing genotype- and stage-dependent chlorophyll, gas-exchange and injury-related changes. [S09] An unqualified “single optimum temperature for sugarcane” is not a meaningful physiological parameter.
4.3 干旱与水汽压亏缺:供给和需求 / Soil water and VPD: supply and demand
土壤缺水降低水分供给,空气VPD增大提高蒸发需求;两者未必同步。 Zhao等盆栽研究在七至八叶期开始控水,记录了气孔导度、净光合、蒸腾和叶面积的下降。 [S01] Silva等在胁迫发展过程中记录到VPD变化,提示测量时必须联合气象与叶水状态。 [S02] Grantz的蓝光脉冲试验说明VPD会影响气孔开启动力学,但不能从短时开启速度推出长期耗水优势。 [S11] 识别水分瓶颈需联测根区体积含水量/水势、叶水势、气孔与蒸腾以及作物年龄。
Soil drying reduces hydraulic supply, whereas increasing atmospheric VPD raises evaporative demand; the two need not change together. In a pot experiment, Zhao and colleagues withheld water at the seven- to eight-leaf stage and reported declining conductance, net photosynthesis, transpiration and leaf area. [S01] Silva and colleagues recorded changes in VPD as stress developed, showing the need to pair weather with leaf water status. [S02] Blue-light pulse experiments demonstrated that VPD affects stomatal opening kinetics, but faster transient opening cannot be converted into a claim of superior seasonal water use. [S11] Diagnose this pathway jointly using root-zone moisture or potential, leaf water potential, stomatal and transpiration measurements, and crop age.
4.4 积水、盐度与养分:根区多重混杂 / Flooding, salinity and mineral supply
土壤淹水改变根区氧和还原环境,也可能伴随养分有效性变化;盐害可通过渗透胁迫、离子失衡及根系生长下降表现。 Zhao等以0、38、75、150和300 mM外加NaCl设盆栽处理,涉及两份商业品种与一份Erianthus材料;这些剂量是处理设计值,不是田间土壤饱和提取液ECe门槛。 [S08] 若试验同时改变施肥、水位与盐分而没有独立对照,观察到的SPAD或茎长差异不能归因给单一因素。
Waterlogging can alter root-zone oxygen and redox conditions together with nutrient availability; salinity can act through osmotic load, ionic imbalance and curtailed root growth. Zhao and colleagues applied nominal NaCl additions of 0, 38, 75, 150 and 300 mM in a pot experiment including two commercial varieties and an Erianthus material; those treatment concentrations are not thresholds for field saturated-paste ECe. [S08] When fertilization, water table and salinity change together without independent controls, a difference in SPAD or stalk length cannot be assigned to one causal factor.
外因 / factor | 应联测的近端变量 / proximal | 不可直接跳到的结论 / not directly inferred |
|---|---|---|
光 / Light | PPFD, leaf rank, photosynthesis light curve | 密植最佳值 / optimum population density |
温 / Temperature | leaf T, Fv/Fm, enzyme/activity assays | 全球温度阈值 / universal threshold |
旱 / Water deficit | θv, Ψleaf, VPD, gs, transpiration | 最终糖减产比例 / final sugar-loss percentage |
涝 / Flood | water-table depth, duration, oxygen, roots | 耐涝绝对排名 / universal tolerance rank |
盐 / Salinity | soil ECe, ion content, leaf water status | 外加mM=田间ECe / nominal dose ≠ field ECe |
养分 / Nutrition | tissue N/K, growth and root supply | 单次SPAD=养分限制 / SPAD alone ≠ causal N deficiency |
五、基因型、生态区与相反证据 / Genotypes, regions and conflicting results
5.1 “耐性”不是一个没有条件的固定排名 / Tolerance is contextual
材料在温室干旱试验中的高气孔导度,可能在有深层可提取水时有利于吸碳,却也可能在供水有限时更快消耗土壤水。 跨三个生产区和多个作物周期的研究发现,气孔导度与蔗产量的遗传相关范围从负值到正值,表明环境改变排名。 [S12] 温室的CP材料、巴西HoCP/TCP材料、印度热胁迫材料、云南高糖品种,不应只因同属甘蔗就被合并为一个“耐逆性”指标。
High stomatal conductance in a greenhouse drought trial may be beneficial when deep extractable water is available but may hasten depletion under a finite seasonal supply. Across three production regions and crop cycles, the genetic correlation between conductance and cane yield ranged from negative to positive, implying that rankings can change across environments. [S12] Canal Point genotypes, Brazilian HoCP/TCP clones, Indian heat-response material and Chinese field light-response varieties should not be merged into a single “stress tolerance” scale merely because all are sugarcane.
5.2 低温反应的材料差异 / Cold-response contrasts
Yomitanzan、NiF4和Badira在同一10°C处理下光合损失和C4酶活性轨迹不同,表明材料背景可改变控制环节。 [S06] 两品种冷处理与复温试验同时测叶绿素荧光和气体交换,提供了另一组独立的短期冷响应证据。 [S13] 然而,不同试验的光强、预培养温度、处理持续期及叶龄并不一致,不能用某个百分比直接给另一品种排序。
Yomitanzan, NiF4 and Badira differed in the trajectories of assimilation and C4-enzyme activities under the same 10°C treatment, showing that genetic background can shift the relevant bottleneck. [S06] A separate two-cultivar chilling-and-rewarming experiment combined chlorophyll fluorescence with gas exchange. [S13] Because irradiance, pre-growth temperature, exposure duration and tissue age differed across experiments, a percentage response in one study should not be transferred as an absolute cultivar ranking in another.
5.3 涝害证据的表面冲突与解释 / The apparent flooding paradox
同一环境因子可以造成不一致的方向:成年植株的四轮短时淹水条件下,光合和蒸腾往往不显著下降,有时反而略增;幼龄植株持续数周的淹水则出现器官生物量减少。 [S03][S04] 前者评价较短时的叶片功能,后者评价长时生物量;加上土壤类型、根系年龄与品种差异,两项研究不构成相互推翻。 证据表必须明确每条结论适用的水位、时长、材料和响应变量。
The same nominal stress can produce differently signed observations: established plants during four short flooding cycles often maintained, and occasionally improved, leaf gas exchange, whereas young cane flooded for weeks lost organ biomass. [S03][S04] One experiment measured relatively immediate leaf function, while the other integrated biomass over much longer exposure. Different soils, root ages and genotypes add further scope limits. The findings are not mutual refutations; claim records must state water depth, duration, material and response variable.
六、原始试验、识别策略和量化框架 / Original experiments, identification and quantitative framework
6.1 实验设计:随机、梯度、互作和恢复 / Design: randomized gradients, interaction and recovery
环境限制诊断优先选择分层随机的环境干预试验,而不是仅按低产地块的土壤照片倒推原因。 推荐最小设计同时考虑至少两个环境水平、适当材料和生育阶段的重复、足够接近的初始株龄,以及分阶段非破坏观测与最终独立小区的破坏性生物量测定。 研究热×旱、盐×水或水位×品种时,完整因子设计比仅两个极端处理更能区分主效应和交互效应。 重复单位是被独立随机施加处理的盆、池或小区;同一盆中的三片叶不等于三次独立重复。
Identification should prioritize randomized environmental interventions rather than post-hoc explanations based on photographs of low-yield fields. At minimum, contrast meaningful environmental levels with replicated genotypes and stages, comparable initial plant age, repeated non-destructive observations and destructive biomass sampling from independent experimental units. For heat × drought, salinity × water or water-table × genotype, a factorial design permits separation of main and interaction effects. The independent unit is the pot, lysimeter or plot assigned a treatment; three leaves from one pot are subsamples, not three independent replicates.
6.2 四种证据强度 / Four strengths of evidence
本书将主张按证据来源与推断距离登记:A为可核读方法和数据位置支持的有限范围结果;B为出版商摘要直接支持但细节待复核;C为机制合理但需要多步骤推断;L为仅有线索。 A级也不意味着全球有效。 以“在12个渗漏计及特定排水周期,叶片气体交换并未一致下降”为B级原文摘要事实;“所有田块淹水均有利于甘蔗”为不成立的越界主张。 原始论文与数据集有共同作者或地点,不自动等于同一试验,但独立性必须进一步核实。
Claims are graded by inspected evidence and inferential distance: A denotes a bounded result supported by inspected methods and result location; B an outcome directly supported in the publisher abstract with unresolved detail; C a plausible but multi-step mechanistic inference; L a lead only. Grade A does not mean globally universal. “Leaf gas exchange did not consistently decline under the specified lysimeter flood cycles” is a bounded abstract-supported claim; “all flooding benefits sugarcane everywhere” is unsupported. Shared authors and facilities do not automatically imply a single experiment, but independence requires explicit investigation.
6.3 基本公式和单位陷阱 / Core calculations and unit pitfalls
可用的基础检验包括:气孔内在水分利用效率iWUE=A/gs,其中A应为CO₂摩尔通量、gs为水汽导度,单位及定义须保持一致;作物生长速率CGR=(W2−W1)/(A地×Δt);单位面积糖产量=鲜蔗产量×测得的可回收糖分数。 以上是定义关系,并非证明环境因果的公式。 VPD应区分叶气与空气值;土壤体积含水量θv(m³·m⁻³)、水势(MPa)及饱和提取液电导率ECe(dS·m⁻¹)不能直接互换。
Useful checks include intrinsic water-use efficiency iWUE = A/gs, with A as molar CO₂ flux and gs as conductance to water vapour and consistent unit conventions; crop growth rate CGR=(W₂−W₁)/(ground area×elapsed time); and recoverable sugar yield=harvested cane mass×measured recoverable-sugar fraction. These are definitions, not identification of environmental causality. Leaf-to-air VPD must be distinguished from ambient VPD; volumetric soil water θv (m³ m⁻³), water potential (MPa) and saturated-extract ECe (dS m⁻¹) are not interchangeable.
6.4 观测矩阵:从近端到远端 / Measurement matrix: from proximal to distal
同一次实验应记录空气温湿度、太阳辐射、叶温、叶位、基质土壤水势或含水量、根区氧指示量、养分状态、气孔导度与蒸腾、净同化和Fv/Fm、叶面积、有效茎数、单位面积干物质、成熟度与最终糖产量。 频率由反应速度决定:气象数据至少日内连续或定时,叶片交换与叶水势须固定取样时段,生物量和糖分需跨阶段采集。 只给“增产率%”而不给绝对值、原始单位、基准对照和误差的研究不应进入可比较的量化汇总。
A coherent study records air temperature and humidity, radiation, leaf temperature and rank, substrate water potential or water content, root-zone oxygen proxies, nutrient status, stomatal conductance, transpiration, net assimilation and Fv/Fm, leaf area, surviving stalk number, area-based dry matter, maturity and final sugar output. Sampling frequency should match response kinetics: weather measurements need temporal resolution; leaf gas exchange and water potential require aligned time windows; biomass and quality must be sampled across developmental phases. A bare percent yield change without an absolute base, treatment definition, units and uncertainty is not eligible for quantitative pooling.
数据字段 / field | 单位或类型 / unit/type | 必须记录的意义 / requirement |
|---|---|---|
source_id, experiment_id | string | 论文与独立试验分开 / separate paper from experiment |
genotype, crop_cycle, stage | string / code | 材料与蔗作周期 / genetic & phenological context |
treatment, control | JSON / controlled text | 随机处理与基线 / treatment and reference |
experimental_unit, n_units | unit; integer/null | 盆/池/小区;未知保留null / pot, lysimeter, plot |
leaf_rank, observation_datetime | int; timestamp | 叶位、日内时段 / position and timing |
A, gs, E, VPD, Ψleaf | typed numeric / null | 原始单位、仪器、误差 / units, methods and errors |
biomass_dry, stalks_m2, sugar_yield | mass/area/time | 绝不从A推算产糖 / never equate A to sugar yield |
source_locator, grade, reuse_relation | strings | 具体原文位置、证据级与关系 / traceability |
七、真实图像证据与数据库结构 / Authentic visual evidence and data schema
7.1 现场照片的有效信息和不足 / What a field photograph can and cannot show
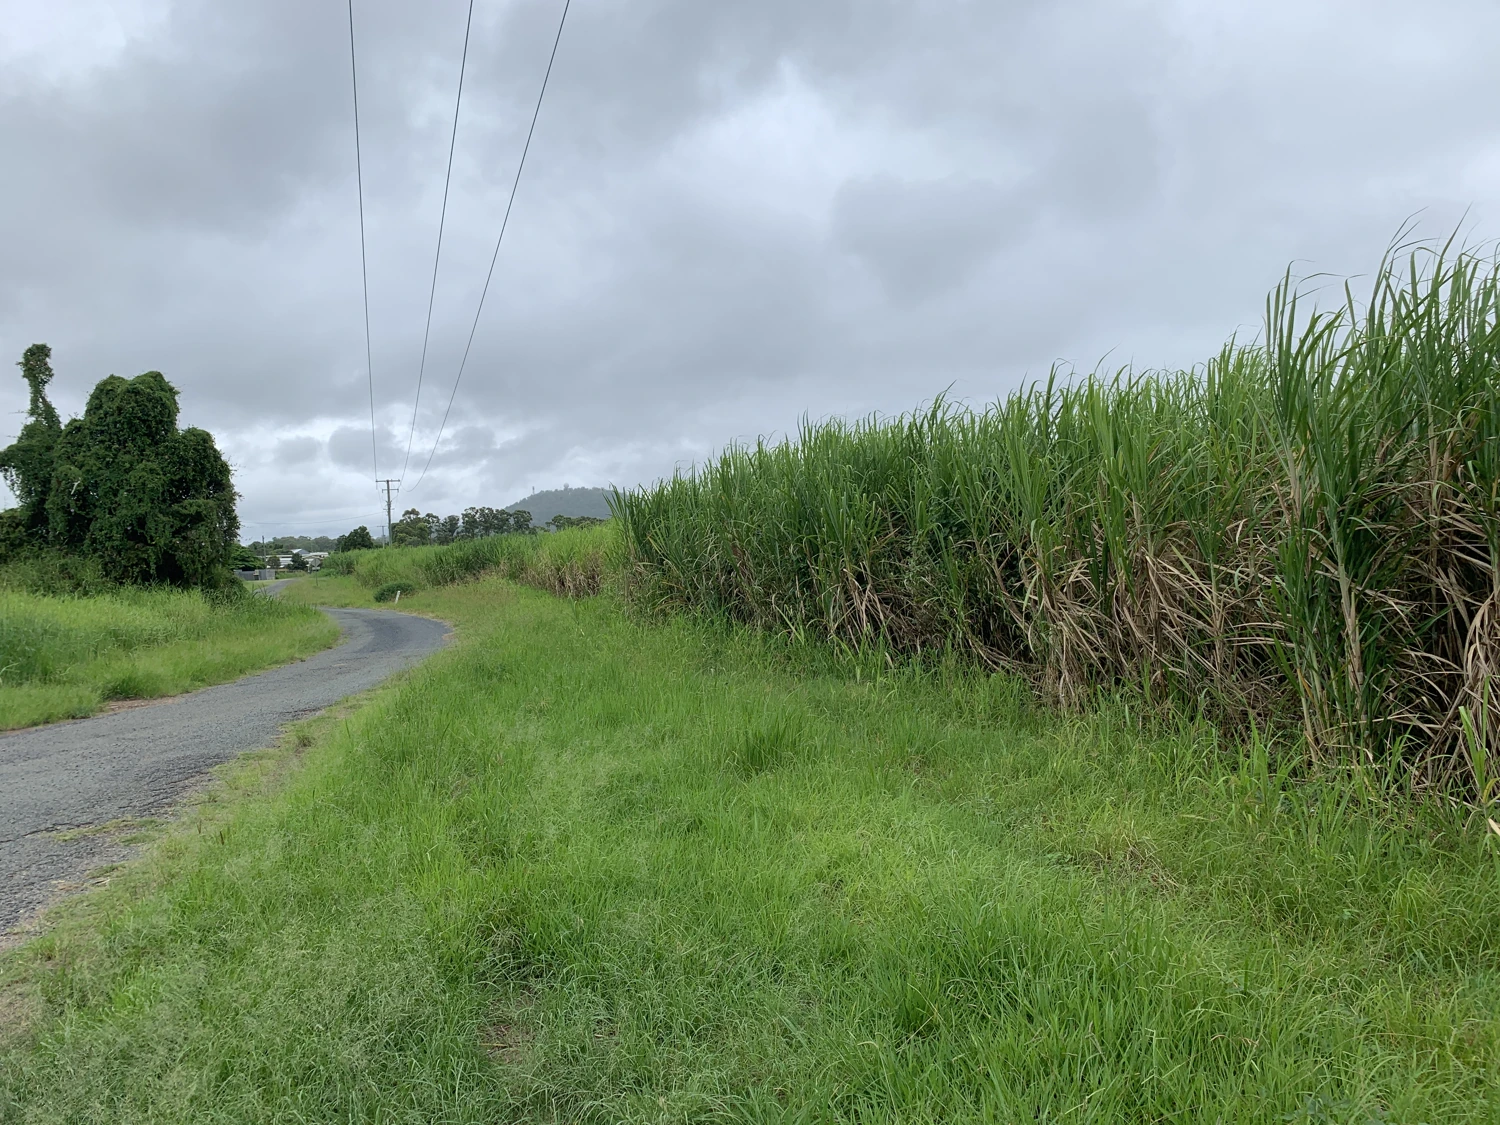
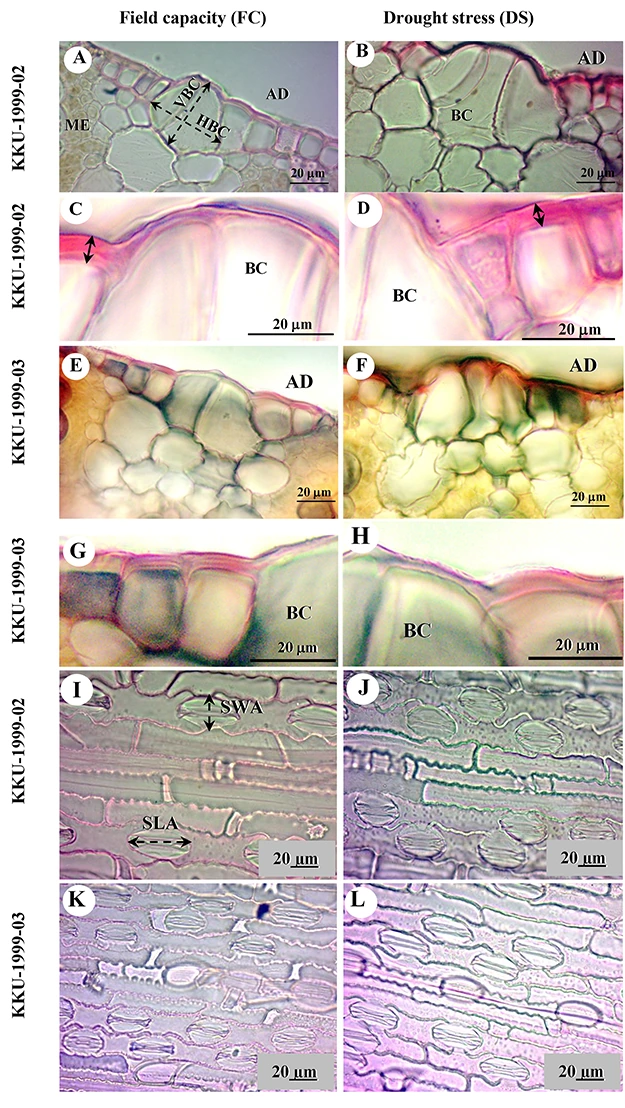
经核验的澳大利亚甘蔗田实拍图用于呈现冠层高度、行间可见度和群体背景;照片本身没有测量土壤水分、VPD、叶温或蔗糖。 另一张真实叶片显微图出自KKU材料的田间持水与干旱对照,可见组织和气孔形态,但不得将其面板上的组织差异写成所有品种在所有干旱环境的普遍规律。 两幅图均为复用的已验证素材,本章不把复用算新增摄影证据。
The verified Australian field photograph documents canopy appearance, visible inter-row structure and field context, not soil moisture, VPD, leaf temperature or sucrose measurements. A second genuine sugarcane leaf micrograph from an experiment contrasting field capacity and drought treatments illustrates epidermal and stomatal anatomy; its visible panel differences are not universal effects for every genotype or drought regime. Both illustrations are reused, previously inspected assets and are not counted as newly acquired photographic evidence.
7.2 原始数据的最小可追溯实体 / Minimum provenance entities
数据库至少拆分为Source(文献)、Study(独立试验)、Treatment(处理)、Unit(随机化单位)、Observation(观测)、Claim(主张)、Media(图像)和Relation(复用或引证关系)。 每条数值除value与unit外,应写明变量类型、原文位置、观测层级、日期/时刻、处理、基准与不确定性;无原始值必须使用null并附原因。 摘要可核实试验处理设计,却不能自动推导方差、样本重复或独立试验数量。
The minimum schema separates Source (publication), Study (independent experiment), Treatment, Unit (randomization unit), Observation, Claim, Media and Relation (data reuse or citation). Each number requires value and unit plus variable class, original location, observation level, date/time, treatment, baseline and uncertainty. Unavailable values remain null with an explicit reason. A publisher abstract can establish treatment design but does not automatically supply variance, replication or a count of distinct independent experiments.
7.3 图片版权、比例尺与双语图注 / Image rights, scale bars and bilingual captions
论文图、新闻现场照、农民自摄和示意图属于不同证据类型。 只有实际取得并查看像素、核对署名与许可、保留原始SHA-256后,才列入“已取得真实图像”。 图中的20微米比例尺是作者对显微照片给出的空间参考;普通田间照片无比例尺不得臆造。 若某幅候选原图下载失败,则保留该线索与失败记录,不换镜像反复下载,也不能因网页出现缩略图就称原件入库。
Research figures, press photographs, farmer photographs and explanatory drawings are distinct evidence categories. An image enters the acquired-authentic collection only after its actual pixels have been inspected, attribution and licence checked, and the original SHA-256 preserved. The original 20 µm bar is a micrograph scale reference; a field photo without a scale bar must not be assigned an invented one. A failed original download remains a lead with its failure recorded, not an acquired image merely because a thumbnail is visible online.
网页预览经过缩放或格式转换,未裁切;原比例尺与标签保留。 / Web preview resized or re-encoded without cropping; original scales and labels retained.
图1 澳大利亚昆士兰Alberton甘蔗田真实照片:用于解释冠层空间结构;非本章生理观测地块。 作者Kerry Raymond,拍摄日期按原页面为2022-01-26。
Figure 1. Authentic sugarcane field in Alberton, Queensland, Australia; a canopy-context image, not a measured physiological treatment plot. Kerry Raymond; original page reports 2022-01-26.
Source / 来源: https://commons.wikimedia.org/wiki/File:Sugarcane_fields,_looking_south_down_Cane_Farm_Road,_Alberton,_2022_01.jpg License / 许可: CC BY 4.0 SHA-256: fc287e4f805052bee0d1a15c308152b87cc5bd804f4ddf208f4b908e72381fb2
网页预览经过缩放或格式转换,未裁切;原比例尺与标签保留。 / Web preview resized or re-encoded without cropping; original scales and labels retained.
图2 原始研究显微图,KKU甘蔗材料在田间持水量(FC)和干旱处理(DS)下的叶缘与表皮,原图分面板A—L,原标尺20 µm;本图不能独立证明群体产量变化。
Figure 2. Original research micrographs of KKU sugarcane leaf margins and epidermis under field-capacity (FC) and drought-stress (DS) treatments; original panels A–L and 20 µm bars. The figure alone does not establish a crop-yield response.
Source / 来源: https://www.journalssystem.com/agb/Leaf-Anatomical-Adaptation-Under-Early-Drought-Stress-of-Sugarcane-Cultivars-KKU,159857,0,2.html License / 许可: CC BY 4.0 SHA-256: 52f7e3126da02d991d0754c4af1d4ecd20272a99e16e1e29a06f44a4e766d008
八、适用边界、开放问题与章节衔接 / Boundaries, unknowns and cross-chapter links
8.1 哪些尚不能下定论 / What remains unresolved
目前没有足够跨地区同口径实测数据来给出甘蔗光、温、旱、涝与盐分的单套全球阈值。 部分来源仅能查看摘要,缺少完整随机化方法、重复数与误差;第009章也没有新增取得真实逆境现场照片。 尤其不能把“短期叶片净光合下降20%”直接当作“最终糖产量下降20%”。 未来应寻找多站点、跨季节、相同品种与记录口径的因子试验,补齐根区连续观测、最终糖产量及开放的逐小区数据。
There is not enough consistently measured multi-region evidence here to prescribe one global threshold for light, temperature, drought, flooding or salinity across sugarcane. Some sources were inspected only at abstract level, leaving randomization, replication and error terms unresolved; this chapter also did not acquire a new authentic stress-field photograph. A 20% short-term reduction in leaf assimilation cannot be re-labelled as a 20% loss of final sugar yield. Future evidence should prioritize replicated multi-site and multi-season factorial studies with shared genotypes and definitions, continuous root-zone measurements, final recoverable sugar and openly available plot-level observations.
8.2 与全书后续章节的关系 / Cross-links within the 180-chapter encyclopedia
本章为第二卷的光合生理、后续卷的水分关系、营养过程、根系生态、分蘖与茎伸长、成熟积糖及复合逆境提供“外因—近端—群体—产量”的共同证据链。 具体灌溉设备和施肥配方不在本章做处方;品种排序不代替育种鉴定;工厂实际提糖率也不与田间Brix混写。 下一章第010章专门讨论表型可塑性、驯化与遗传适应,延伸本章关于胁迫历史与恢复的观察,严格区分同一个体可逆改变和跨代遗传改变。
This chapter supplies a shared exposure–proximal process–crop integration–yield logic for subsequent chapters on photosynthesis, water relations, nutrient physiology, root ecology, tillering and elongation, ripening and combined stresses. Irrigation hardware and fertilizer prescriptions belong to the applied companion encyclopedias; cultivar ranking does not replace breeding evaluation; factory sugar recovery must not be conflated with field Brix. Chapter 010 takes forward plasticity, acclimation and genetic adaptation, distinguishing reversible changes in one plant from heritable change across generations.
附录 A|可反驳的研究假说 / Appendix A: Falsifiable research hypotheses
H09-A:在温度和光照接近的条件下,分期控水引起的叶水势与气孔变化应先于绿色叶面积和干物质的改变;否则该顺序假说不成立。
H09-A: At comparable light and temperature, changes in water potential and stomata should precede changes in green area and dry matter during imposed drought; otherwise the proposed order fails.
H09-B:同品种不同生长阶段对相同短期淹水的响应强度不同,根系年龄与已有通气组织可部分解释差异;需要直接测根氧和生物量。
H09-B: Response to the same short flood differs by crop stage, partly associated with root age and aerenchyma; direct root oxygen and biomass measurements are required.
H09-C:升高VPD在土壤持水充足与供水受限背景下,对气孔、叶温与生物量具有不同方向或幅度的效应;需要VPD×灌溉因子试验。
H09-C: Raising VPD may have different effects on conductance, leaf temperature and biomass under ample versus limited root supply; a VPD × irrigation factorial test is required.
H09-D:相同外加NaCl浓度下,不同基质与浇灌方式产生的实测ECe不同,因此名义盐浓度无法作为普适根区盐胁迫尺度。
H09-D: Identical nominal NaCl additions can produce different measured ECe in different media or irrigation schedules; nominal dose is not a universal root-zone stress scale.
H09-E:同叶光合反应不一定预测单位面积产糖,除非有冠层截光、秆数、干物质分配及成熟品质的独立观测。
H09-E: A leaf-assimilation response need not predict sugar yield per area without independent canopy interception, stalk population, dry-matter allocation and maturity assays.
附录 B|中英双语术语 / Appendix B: Chinese–English terminology
中文术语 / Chinese | 英文术语 / English |
|---|---|
环境因子 | Environmental factor |
限制因素 | Limiting factor |
限制步骤 | Limiting step |
共同限制 | Co-limitation |
近端生理指标 | Proximal physiological indicator |
可检验假说 | Testable hypothesis |
气孔导度 | Stomatal conductance (gs) |
净光合速率 | Net assimilation rate (A) |
蒸腾速率 | Transpiration rate (E) |
叶气水汽压亏缺 | Leaf-to-air vapour pressure deficit (VPD) |
叶水势 | Leaf water potential |
根区缺氧 | Root-zone hypoxia |
土壤体积含水量 | Volumetric soil water content |
饱和提取液电导率 | Saturated-paste electrical conductivity (ECe) |
光合有效辐射 | Photosynthetically active radiation (PAR) |
光合光量子通量密度 | Photosynthetic photon flux density (PPFD) |
光抑制 | Photoinhibition |
叶绿素荧光 | Chlorophyll fluorescence |
光系统II最大量子效率 | Maximum PSII efficiency (Fv/Fm) |
低温胁迫 | Chilling stress |
热胁迫 | Heat stress |
胁迫恢复 | Stress recovery |
暴露历时 | Exposure duration |
遗传相关 | Genetic correlation |
新植蔗 | Plant cane |
宿根蔗 | Ratoon cane |
试验单位 | Experimental unit |
亚样本 | Subsample |
因子设计 | Factorial design |
主效应 | Main effect |
交互效应 | Interaction effect |
干物质积累 | Dry-matter accumulation |
糖产量 | Recoverable sugar yield |
证据边界 | Evidence boundary |
附录 C|原始研究索引 / Appendix C: Primary research index
[S01] D. Zhao; B. Glaz; J. C. Comstock (2013). Sugarcane Leaf Photosynthesis and Growth Characters during Development of Water-Deficit Stress. Crop Science 53:1066–1075. DOI: 10.2135/cropsci2012.09.0554. Access scope / 已核读范围: PUBLISHER_ABSTRACT. https://acsess.onlinelibrary.wiley.com/doi/abs/10.2135/cropsci2012.09.0554
[S02] M. de Almeida Silva; J. L. Jifon; C. M. dos Santos; C. J. Jadoski; J. A. G. da Silva (2013). Photosynthetic capacity and water use efficiency in sugarcane genotypes subject to water deficit during early growth phase. Brazilian Archives of Biology and Technology 56(5). DOI: 10.1590/S1516-89132013000500004. Access scope / 已核读范围: PUBLISHER_FULL_HTML. https://www.scielo.br/j/babt/a/jzBcSWs3K7jHj67wKXpQxNn/?lang=en
[S03] B. Glaz; D. R. Morris; S. H. Daroub (2004). Sugarcane Photosynthesis, Transpiration, and Stomatal Conductance Due to Flooding and Water Table. Crop Science 44:1633–1641. DOI: 10.2135/cropsci2004.1633. Access scope / 已核读范围: PUBLISHER_ABSTRACT. https://acsess.onlinelibrary.wiley.com/doi/abs/10.2135/cropsci2004.1633
[S04] B. Glaz; S. E. Lingle (2012). Flood Duration and Time of Flood Onset Effects on Recently Planted Sugarcane. Agronomy Journal 104:575–583. DOI: 10.2134/agronj2011.0351. Access scope / 已核读范围: PUBLISHER_ABSTRACT. https://acsess.onlinelibrary.wiley.com/doi/10.2134/agronj2011.0351
[S05] B. Glaz; D. R. Morris (2010). Sugarcane Responses to Water-Table Depth and Periodic Flood. Agronomy Journal 102:372–380. DOI: 10.2134/agronj2009.0262. Access scope / 已核读范围: PUBLISHER_ABSTRACT. https://acsess.onlinelibrary.wiley.com/doi/abs/10.2134/agronj2009.0262
[S06] Y.-C. Du; A. Nose; K. Wasano (1999). Effects of chilling temperature on photosynthetic rates, photosynthetic enzyme activities and metabolite levels in leaves of three sugarcane species. Plant, Cell & Environment 22:317–324. DOI: 10.1046/j.1365-3040.1999.00415.x. Access scope / 已核读范围: PUBLISHER_FULL_HTML. https://onlinelibrary.wiley.com/doi/full/10.1046/j.1365-3040.1999.00415.x
[S07] D. F. S. P. Machado; A. M. M. A. Lagôa; R. V. Ribeiro; P. E. R. Marchiori; R. S. Machado; E. C. Machado (2013). Low night temperature and water deficit on photosynthesis of sugarcane. Pesquisa Agropecuária Brasileira 48(5):487–495. DOI: 10.1590/S1678-3921.pab2013.v48.14406. Access scope / 已核读范围: PUBLISHER_ABSTRACT. https://apct.sede.embrapa.br/pab/en/article/view/14406
[S08] D. Zhao; K. Zhu; A. Momotaz; X. Gao (2020). Sugarcane Plant Growth and Physiological Responses to Soil Salinity during Tillering and Stalk Elongation. Agriculture 10(12):608. DOI: 10.3390/agriculture10120608. Access scope / 已核读范围: PUBLISHER_ABSTRACT_SEARCH_INDEX. https://www.mdpi.com/2077-0472/10/12/608
[S09] S. Kohila; R. Gomathi (2018). Adaptive physiological and biochemical response of sugarcane genotypes to high-temperature stress. Indian Journal of Plant Physiology 23:245–260. DOI: 10.1007/s40502-018-0363-y. Access scope / 已核读范围: PUBLISHER_FULL_HTML. https://link.springer.com/article/10.1007/s40502-018-0363-y
[S10] Y. Y. Liu et al. (2020). Sugarcane leaf photosynthetic light responses and their difference between varieties under high temperature stress. Photosynthetica 58(4):1009–1018. DOI: 10.32615/ps.2020.038. Access scope / 已核读范围: PUBLISHER_ABSTRACT. https://ps.ueb.cas.cz/artkey/phs-202004-0013_sugarcane-leaf-photosynthetic-light-responses-and-their-difference-between-varieties-under-high-temperature-str.php
[S11] D. A. Grantz (1990). Stomatal response to humidity in sugarcane and soybean: effect of vapour pressure difference on the kinetics of the blue light response. Plant, Cell & Environment. DOI: 10.1111/j.1365-3040.1990.tb01288.x. Access scope / 已核读范围: PUBLISHER_ABSTRACT. https://onlinelibrary.wiley.com/doi/abs/10.1111/j.1365-3040.1990.tb01288.x
[S12] J. Basnayake; P. A. Jackson; N. G. Inman-Bamber; P. Lakshmanan (2015). Sugarcane for water-limited environments. Variation in stomatal conductance and its genetic correlation with crop productivity. Journal of Experimental Botany 66(13):3945–3958. DOI: 10.1093/jxb/erv194. Access scope / 已核读范围: PUBLISHER_ABSTRACT_AND_INTRODUCTION. https://academic.oup.com/jxb/article/66/13/3945/515539
[S13] S. Mathur; V. S. J. Sunoj; N. I. Elsheery; V. R. Reddy; A. Jajoo; K.-F. Cao (2021). Regulation of Photosystem II Heterogeneity and Photochemistry in Two Cultivars of C4 Crop Sugarcane Under Chilling Stress. Frontiers in Plant Science 12:627012. DOI: 10.3389/fpls.2021.627012. Access scope / 已核读范围: PUBLISHER_FULL_HTML. https://www.frontiersin.org/journals/plant-science/articles/10.3389/fpls.2021.627012/full
附录 D|证据冲突与跨尺度核对表 / Appendix D: Contradictions and scale checks
下表不是额外试验结果,而是后续编辑必须逐项查证的证据边界。
The following are editorial decision rules, not additional experimental results.
待核命题 / proposition | 关键反证或边界 / counter-evidence or limit | 后续核实路径 / verification |
|---|---|---|
淹水总会降低光合 / Flood always reduces A | 短周期成年蔗结果可为中性或正向 [S03] / Short floods did not consistently depress A | 根区氧、暴露时长、生育期 / O₂, duration, stage |
长期淹水都无害 / All long floods harmless | 幼龄蔗0–6周生物量损失 [S04] / Young plants lost biomass | 重复独立盆/池及冠层重量 / replicated pots and biomass |
高导度一定高产 / Higher gs always means more yield | rg在-0.29~0.94之间 [S12] / correlation crosses zero | 分区域与水分状态分析 / stratify region & water |
低温只限制气孔 / Cold limits only stomata | C4酶响应不同 [S06] / enzyme changes also differ | 同叶A–Ci和酶/荧光 / matched A–Ci, enzymes, PSII |
盐处理mM等于田间ECe / NaCl dose equals ECe | 盆栽外加量≠土壤提取量 [S08] / dose is not measured ECe | 配套ECe与离子测定 / measured ECe and ions |
叶片下降20%=糖产量下降20% / A loss = sugar loss | 不同时间与尺度 / multiple temporal and spatial scales | 独立产量小区与回收糖 / plot yield and sugar recovery |
网页配图即已取证 / Thumbnail counts as acquired photo | 原始文件未取得时不能计算SHA / No SHA without file | 像素、版权、文件哈希 / pixels, licence, SHA-256 |
方法声明:对每条主张,保留支持证据与不支持的条件;在没有与试验单位对应的方差与原始观测时,不做跨研究效应量合并。
Methods statement: preserve both support and exceptions for every claim. Without variance and observations linked to independent experimental units, no pooled cross-study effect size is computed.
编写状态 / Editorial and release status
已形成双语正文及逐项证据初稿;需要继续核对部分原始全文、随机化和误差、不同站点的独立性以及后续可合法获得的环境胁迫现场照片。 完整180章通过统一核查后方可打包;本章不直接发布GAKI网站。
Bilingual chapter draft and claim-level evidence ledger compiled. Full-method verification, independent units, variance and availability of licensed stress-field imagery remain open. No website deployment or whole-book package is authorized before all 180 chapters pass unified review.