GAKI-SUG-PHY-V01-C004 | R1 · 2026-11-09 | 双语研究初稿与首轮原始证据核查 / Bilingual draft and initial primary-evidence review
S01 研究对象与核心问题 / Objects and key questions
1.1 五级对象及其研究单位 | 1.1 Five levels and observational units
中文|甘蔗生理生态不是将细胞、叶片、茎、植株和田块的测量值相加,而是研究过程如何在不同空间和时间尺度之间耦合。 本章采用细胞/亚细胞、组织、器官、单株/分蘖群体、田间群体五级框架。 细胞尺度关注叶绿体容积、胞间连丝、酶活性;组织尺度关注叶肉与维管束鞘协作、维管输送和薄壁细胞储糖;器官尺度涉及叶片、节间和根;单株尺度考虑叶龄与库源联系;田块尺度才计算面积截光、干物质和蔗糖产出。 每一级的“测量对象”“独立试验单位”和“统计总体”须分开登记。 [S01,S02,S03]
English|Sugarcane ecophysiology does not simply add measurements from cells, leaves, culms, plants and fields. It explains how mechanisms couple across space and time. This chapter distinguishes subcellular/cellular, tissue, organ, plant/tiller and field-canopy levels. Chloroplast geometry and enzyme activity are cellular traits; mesophyll–bundle-sheath cooperation, vascular transport and storage parenchyma are tissue processes; leaves, internodes and roots are organs. Whole-plant source–sink coordination and canopy interception require distinct observational units. For each level the object measured, independently replicated unit and population of inference must be recorded separately. [S01,S02,S03]
1.2 统计尺度与生物学尺度不等价 | 1.2 Statistical scale is not biological scale
中文|一幅显微图可显示数百个叶绿体,但不能据此宣称获得数百株独立甘蔗。 2023年三维叶片研究从3株甘蔗取叶,量取19个维管束鞘叶绿体和242个叶肉叶绿体;这两个数字描述细胞器而不是生物学重复数。 2015年叶片分段研究对4株植株的RNA采用配对比较,叶段样本也不能直接视作独立植株。 将大量细胞、叶段或相机视野直接当作田间独立重复,会造成伪重复并夸大证据精度。 [S01,S02]
English|A micrograph can contain hundreds of chloroplasts without representing hundreds of independently grown plants. In a 2023 3-D anatomy experiment, three sugarcane plants supplied leaves, while 19 bundle-sheath and 242 mesophyll chloroplasts were measured. The latter numbers describe organelles, not biological replicates. In a 2015 leaf-gradient study, RNA measurements from four plants were compared using a paired design; leaf segments were not independent plants. Treating cells, segments or images as experimental replicates creates pseudoreplication and overstates precision. [S01,S02]
1.3 本章要解释的六种转换 | 1.3 Six scale transitions to explain
中文|本章围绕六种转换建立证据链:(一)细胞结构如何约束C4碳浓缩;(二)单片叶沿叶长不同区段如何形成光合功能梯度;(三)叶面积光合如何变成冠层净碳增益;(四)不同节间组织如何分配蔗糖;(五)根系局部吸收如何影响全株水分状态;(六)这些过程如何通过群体密度、光分布及发育阶段改变单位地表面积产量。 每一次跨尺度转换都必须有中介变量,不能用一个尺度的相关性直接证明另一尺度的因果。 [S01–S08]
English|Six transitions organize the evidence: cellular geometry to C4 carbon concentration; longitudinal leaf development to local photosynthetic capacity; leaf-area assimilation to canopy net carbon gain; internode tissue metabolism to sucrose storage; localized root uptake to whole-plant water status; and architecture, density and age to yield per unit land area. Each scale transition requires an explicit intermediate variable. A correlation at one scale does not itself establish causation at another. [S01–S08]
S02 结构基础与过程机制 / Structural basis and process mechanisms
2.1 维管束鞘—叶肉的C4功能分工 | 2.1 C4 cooperation between bundle sheath and mesophyll
中文|甘蔗属于C4植物。 叶肉细胞首先通过磷酸烯醇式丙酮酸羧化酶(PEPC)固定无机碳,C4酸随后进入维管束鞘细胞释放CO₂,Rubisco所处微环境因此获得较高CO₂浓度。 糖生成与转运则同时受光反应能量、叶肉—维管束鞘代谢物通量和胞间连丝连接条件限制。 Laetsch与Price早期观察到维管束鞘与叶肉叶绿体形态不同;Lee等进一步以三维显微观察量化叶绿体体积和胞间连丝壁孔域。 两项研究揭示结构条件,但都不自动证明叶绿体越大就可带来更高吨蔗产量。 [S01,S07]
English|Sugarcane uses C4 photosynthesis. Mesophyll phosphoenolpyruvate carboxylase (PEPC) initially fixes inorganic carbon; C4 acids pass to bundle-sheath cells and release CO2 near Rubisco. The effectiveness of this mechanism depends on energy supply, intercellular metabolite flux and cytoplasmic connectivity. Early microscopy distinguished the two chloroplast types; subsequent three-dimensional imaging quantified chloroplast volume and plasmodesmata pit-field area. These experiments establish a structural substrate, not a demonstration that larger chloroplasts necessarily increase tonnes of harvested cane. [S01,S07]
2.2 三维结构、通量和制样偏差 | 2.2 Three-dimensional geometry, flux and preparation bias
中文|Lee等对CPCL02-0926的维管束鞘叶绿体报告平均体积86.2±6.5 μm³,对叶肉叶绿体报告30.3±0.8 μm³;“±”为文献列明的标准误。 固定、脱水和包埋可以造成收缩,原文也发现激光共聚焦与连续切片电镜所得尺寸差异。 因而这些值是特定制样技术的测量汇总,不能作为活体真实体积的普遍恒定值。 胞间连丝孔域面积亦不等于实际单分子运输速率;只有配合通透性、浓度梯度、转运蛋白及同位素示踪才能估计通量。 [S01]
English|For cultivar CPCL02-0926, Lee et al. reported mean bundle-sheath chloroplast volume of 86.2 ± 6.5 μm³ and mesophyll chloroplast volume of 30.3 ± 0.8 μm³, with uncertainty described as standard error. Fixation, dehydration and embedding can shrink tissue, and serial block-face electron microscopy and laser scanning microscopy produced divergent estimates. These published summaries are method-conditioned measurements, not universal live-cell constants. Similarly, plasmodesmata pit-field area is not itself molecular transport flux: permeability, gradients, transport kinetics and tracer validation are required. [S01]
2.3 叶片内的发育镶嵌体 | 2.3 A developmental mosaic within one leaf
中文|甘蔗叶片不是均匀光合板。 Mattiello等以SP80-3280第一片露出叶领的叶(+1叶)划分基部零段B0、基部B、中部M和叶尖T。 中段较高PEPC活性与光合潜力、不同叶段氮和糖浓度共同说明同一叶片各区段存在发育异质性;但该研究的气体交换只测了B和M,B0与T由于测量腔限制没有直接气体交换结果。 把整叶光合均值赋给每一叶段会掩盖发育梯度;反过来将M段测量外推整个冠层也不成立。 [S02]
English|A sugarcane blade is not a uniform photosynthetic panel. Mattiello et al. divided the first leaf with an exposed dewlap (+1) of SP80-3280 into basal-zero (B0), basal (B), middle (M) and tip (T) segments. Contrasting PEPC activity, nitrogen, sugars and photosynthetic traits demonstrate spatial developmental heterogeneity. Crucially, intact-leaf gas exchange was recorded only at B and M; chamber constraints precluded corresponding B0 and T measurements. Assigning an identical rate to every segment hides the gradient, whereas extrapolating the middle segment to an entire canopy is equally invalid. [S02]
2.4 叶—茎蔗糖运输与贮藏组织 | 2.4 Leaf-to-stem allocation and storage tissues
中文|叶片输出蔗糖经筛管运输至生长点、根、分蘖芽与茎秆节间。 蔗糖在节间中的积累是卸载、合成、裂解、液泡隔离和呼吸的净结果,而不是简单由单叶光合瞬时速率决定。 Schäfer等研究N19第三至第九节间,发现蔗糖合酶出现在维管组织和贮藏薄壁组织,幼嫩与成熟节间的酶表达及反应方向比例不同;随后针对Q117不同年龄节间的代谢谱亦显示组织成熟伴随多类中间代谢物变化。 由于发育位置与器官组织组成相互关联,应避免将“第九节间”的一项酶比值视作每个品种统一的成熟标志。 [S05,S08]
English|Photoassimilated sucrose is exported through phloem to growing apices, roots, tiller buds and internodes. Accumulation in an internode reflects the balance of unloading, synthesis, cleavage, vacuolar sequestration and respiration, rather than instantaneous leaf assimilation alone. In cultivar N19, sucrose synthase was localized in both vascular and storage parenchyma tissues across internodes 3–9, with strong developmental variation in enzyme properties. Metabolite profiling of differently aged Q117 stem regions likewise identified developmental shifts in metabolite pools. Internode number and biochemical ratio must not be promoted into universal markers of maturity. [S05,S08]
2.5 根系的吸收层次和反馈 | 2.5 Root uptake hierarchy and feedback
中文|根尖、根毛区、皮层和木质部具有不同功能。 局部根长密度与接触土体积影响获取水分及养分的机会,但水分进入单根后仍需通过根系导水和茎部水力通路,最终受叶片蒸腾驱动。 巴西第一季宿根甘蔗的根箱试验显示,三种材料在壤质和砂质基质中的根长分布响应并不一致。 根箱提供空间分布证据,但侧壁效应、容器体积和试验环境限制其外推为大型田块的实际取水深度。 [S06]
English|Root tips, root hairs, cortex and xylem contribute differently to resource acquisition. Local root-length density affects the opportunity for water and nutrient uptake, but uptake must still pass through radial and axial hydraulic pathways before coupling with transpiration. A Brazilian first-ratoon rhizotron experiment found cultivar-specific root-length responses to loamy versus sandy substrates. Rhizotrons offer spatial evidence, but wall effects, confinement and controlled conditions prevent direct inference about water extraction depth in extensive fields. [S06]
S03 生育阶段与环境响应 / Developmental stages and environmental responses
3.1 发育阶段是跨尺度模型的时间坐标 | 3.1 Development is the time coordinate of scale bridging
中文|叶芽萌发、叶片展开、茎伸长和成熟并不同步。 发育早期,新生叶和根是竞争库;旺长期扩大叶面积并加强茎秆伸长;后期叶片衰老、蔗糖贮藏和宿根芽准备逐渐改变源库关系。 不同年龄节间代谢物浓度不能单独解释为环境处理效应;对照时必须匹配节位、品种、采样时刻、叶位及水分状态。 本章将每条观测同时登记时间尺度(瞬时、昼夜、周、物候期)和空间尺度。 [S02,S05,S08]
English|Bud sprouting, leaf expansion, internode elongation and ripening are not synchronous. Early in development, young leaves and roots are competing sinks; during grand growth, leaf area and stem elongation expand; later, leaf senescence, storage and ratoon-bud preparation reshape source–sink relations. Metabolic differences among internodes cannot simply be attributed to an environmental treatment unless rank, cultivar, time and water status are controlled. Every observation therefore requires both a temporal scale (instant, diurnal, weekly or phenological) and a spatial scale. [S02,S05,S08]
3.2 光的冠层再分配 | 3.2 Redistribution of light within the canopy
中文|在密植或高大冠层中,上层叶首先截获大量光合有效辐射,下层叶的光照则受行距、叶角、叶面积、叶宽、叶片衰老与太阳角度影响。 Marchiori等对巴西三品种分别测量上、下冠层的日变化气体交换,发现上层CO₂同化相近,而下层光照与IACSP95-3028的生长响应有联系。 因而“最佳叶角”取决于高度层和群体,而非单片叶角越平越好;研究虽有田间材料,其摘要未给出重复小区数,不能擅自填入。 [S04]
English|In tall dense stands, upper leaves intercept much of incoming photosynthetically active radiation while lower leaves depend on row arrangement, leaf angle, leaf area, senescence and solar geometry. Marchiori et al. measured diurnal gas exchange at two canopy positions in three Brazilian cultivars. Upper-canopy CO2 assimilation was similar, whereas differences in lower-canopy light availability were associated with growth of IACSP95-3028. An optimal leaf angle is thus conditional on canopy layer and stand geometry, not a property of one blade in isolation. The accessible abstract does not establish the number of independent field plots; that value remains unknown. [S04]
3.3 水分与温度影响多层过程 | 3.3 Water and temperature act at multiple levels
中文|干旱首先可改变细胞膨压、气孔导度和叶片扩展速率,继而降低冠层面积与蒸腾;极端高温可能同时改变酶动力学、呼吸消耗、叶温与生殖阶段。 一个品种在短期气体交换中的优势,不代表多月的干物质积累与糖分表现必然有优势。 测量需区分瞬时叶面净同化率、日净碳交换、冠层截光、全季节生物量及糖产量。 若不能匹配土壤水分和作物年龄,跨试验比较仅能作为线索。 [S02,S03,S04]
English|Drought may initially alter cell turgor, stomatal conductance and expansion, then reduce canopy area and transpiration. High temperature can simultaneously influence enzyme kinetics, respiratory costs and leaf temperature. A cultivar advantage in a short gas-exchange window need not persist in season-long biomass or sucrose yield. Measurements must distinguish instantaneous leaf net assimilation, daily canopy exchange, intercepted light, season-integrated dry mass and sugar yield. Cross-study comparisons without matching crop age and soil-water status are leads, not calibrated effect estimates. [S02,S03,S04]
S04 品种及生态区差异 / Genotypic and ecological differences
4.1 明确材料而非“甘蔗统一值” | 4.1 Cultivars, not a single sugarcane constant
中文|CPCL02-0926的三维结构、SP80-3280的叶片分段、N19的节间酶定位、Q117的节间代谢谱,以及IACSP三品种的田间冠层均来自不同材料与研究设计。 它们能够构成机制互补,却不能被视为同一品种的连续测量。 育种目标还受品种宿根性、成熟期、抗倒伏和环境适应约束。 章内对每条结论标明材料,缺失材料时明确为null。 [S01,S02,S04,S05,S08]
English|The 3-D anatomy of CPCL02-0926, leaf gradients of SP80-3280, internode enzyme localization in N19, metabolite profiles in Q117 and canopy observations in three IACSP cultivars arise from different genotypes and designs. They supply complementary mechanisms but cannot be joined as a longitudinal dataset from one cultivar. Breeding decisions also depend on ratooning, maturity, lodging and environmental adaptation. Every empirical claim therefore records its material, or null where unresolved. [S01,S02,S04,S05,S08]
4.2 生态区必须落实到可测环境 | 4.2 Ecological zones require measured drivers
中文|所谓“热带”“亚热带”“雨养”“灌溉”只是背景标签,不足以解释生理差异。 可比较的生态记录至少应包括纬度、播种及收获日期、气温与叶温、太阳辐射、土壤类别、根层可利用水、降雨与灌溉时序、株行距、氮供应及作物类型(新植或宿根)。 巴西根箱结果提示品种×基质互作;但根箱的“砂质”不等同于世界各地砂壤土的统一水力属性。 [S04,S06]
English|Labels such as tropical, subtropical, rainfed and irrigated do not by themselves explain physiology. Comparable records should include latitude, crop dates, air and leaf temperatures, solar radiation, soil class, available root-zone water, rainfall and irrigation time series, spacing, nitrogen and plant-cane versus ratoon status. The Brazilian rhizotron study points to genotype × substrate interaction, but its sandy substrate is not a universal hydraulic representation of all sandy soils. [S04,S06]
S05 原始试验与相反证据 / Original experiments and conflicting evidence
5.1 三维显微结构:有重复层级但不代表群体 | 5.1 Three-dimensional imaging: nested measurements, not field inference
中文|Lee等(2023)在玻璃温室用CPCL02-0926节段繁殖,约12周时从3株取最年轻完全展开叶;连续切片电镜分析19个维管束鞘叶绿体和242个叶肉叶绿体。 研究还指出样品收缩和两种成像法的差异。 这直接支持“叶绿体大小因细胞类型而异”,但没有直接测量该品种田间蔗产量,也没有通过独立多地点试验证明结构改造增产。 独立生物单位是取样植株,不是叶绿体数。 [S01]
English|Lee et al. (2023) propagated CPCL02-0926 from nodes in a glasshouse and sampled the youngest fully expanded leaves from three 12-week-old plants. Serial block-face microscopy analyzed 19 bundle-sheath and 242 mesophyll chloroplasts, alongside a method comparison that revealed possible preparation shrinkage. This directly supports differences in organelle geometry between cell types, but does not measure field cane yield or demonstrate yield gains through anatomical manipulation. Plants—not organelles—are the independent biological units. [S01]
5.2 叶片分段试验:相邻组织的配对优势与限制 | 5.2 Leaf segmentation: paired observations and their limits
中文|Mattiello等(2015)使用温室SP80-3280,划分同一片+1叶为B0/B/M/T,并对植株间RNA重复进行配对统计;原文记录RNA有4个独立重复,若干生化图则各有n=4或n=5。 中部叶段的PEPC活性和光合特征较突出,但叶基与叶尖没有直接叶室气体交换。 其跨物种比较引用已有玉米数据集,所以不属于独立产生的玉米实测新试验。 该研究提供器官内部梯度证据,尚不能直接给出整个成熟田间冠层的光合总量。 [S02]
English|Mattiello et al. (2015) examined SP80-3280 in a greenhouse, dividing each +1 leaf into B0/B/M/T and analyzing RNA with a paired design across four independent biological replicates. Selected biochemical figures use n = 4 or n = 5. The middle segment was prominent in PEPC activity and photosynthetic traits, but direct chamber gas exchange was unavailable for the basal-zero and tip segments. Their maize comparison reused a published maize dataset, not a new independent maize experiment. This is convincing evidence for within-leaf gradients, not a direct measurement of net photosynthesis by a mature field canopy. [S02]
5.3 高单叶光合与高产量并不等价 | 5.3 High leaf assimilation does not entail high yield
中文|Irvine(1975)指出单叶单位面积光合速率未随高产品种而一致增加,而叶面积指数与部分试验的蔗吨产量相关;叶排列与含糖表现仅在一项试验中相关,在另一项未重复。 这一“反例”限制了以单叶最高气体交换速率直接筛选高产材料的推断。 另一方面,Marchiori等(2010)报告特定品种下层冠层受光改善与生长相关,两种结果并不矛盾:分别强调的是单叶瞬时速率与群体空间光分配。 [S03,S04]
English|Irvine (1975) reported that leaf-area-based photosynthetic rates did not consistently rise with higher-yielding varieties, whereas leaf-area index was positively related to tonnage in selected tests. Leaf arrangement related to sugar per tonne in one test but not another. This contrary result limits selection based on maximum individual-leaf gas exchange. Marchiori et al. (2010), by contrast, associated better lower-canopy illumination with growth in a particular cultivar. The findings are compatible because they address different causal pathways: instantaneous leaf capacity versus spatial distribution of absorbed light in stands. [S03,S04]
5.4 茎秆与根系证据:组织相关不能替代流量测定 | 5.4 Culm and root evidence: localization is not flux
中文|Schäfer等(2004)以N19节间提取和免疫组织化学显示SuSy在维管组织、储藏薄壁细胞均有定位,并报告裂解与合成活性比由第三节间的约0.12变化为第九节间的约1.4,属于所用检测条件下发表的汇总。 Ido等(2006)比较三品种在两种基质根箱中的根长分布,材料为第一季宿根。 二者均为组织尺度的重要证据,但前者未直接测蔗糖运输净流量,后者未测整田根系水分吸收;“酶有定位”“根长较多”均不能自动改写为“糖产量较高”或“水分利用效率较高”。 [S05,S06]
English|Schäfer et al. (2004) localized sucrose synthase in vascular and storage parenchyma of N19 internodes and reported an activity-direction ratio increasing from about 0.12 in internode 3 to about 1.4 in internode 9 under their assays. Ido et al. (2006) compared root-length distributions for three first-ratoon cultivars in two rhizotron substrates. Both are valuable tissue-level evidence, but the former did not measure net sucrose export directly, and the latter did not quantify whole-field water extraction. Enzyme localization and root length cannot automatically be relabeled as superior sugar yield or water-use efficiency. [S05,S06]
表 004-1:原始研究与独立单位 / Table 004-1: Original research and independent units
ID | Study / 研究 | Independent sampling / 单位 | Read scope / 核读范围 |
|---|---|---|---|
S01 | Lee 2023 | 3 plants / 19 BS + 242 M chloroplasts | Full HTML; nested organelles |
S02 | Mattiello 2015 | 4 independent RNA plants; figures n=4/5 | Full HTML; paired segments |
S03 | Irvine 1975 | Field plot n unknown | Publisher abstract |
S04 | Marchiori 2010 | 3 cultivars; plot n unknown | Bibliographic abstract |
S05 | Schäfer 2004 | N19, internodes 3–9; plant n unknown | Publisher abstract |
S06 | Ido 2006 | 3 cultivars × 2 substrates; unit n unknown | Publisher abstract |
S06 观测指标与测量方法 / Variables and measurement methods
6.1 构建带单位的跨尺度观测链 | 6.1 Build unit-aware scale bridges
中文|细胞层登记叶绿体容积(μm³)、胞间连丝孔域面积(μm²)和酶活性(明确鲜质量、蛋白量或面积分母);组织与器官层登记叶绿素、总氮、叶片净同化率A(μmol CO₂ m⁻²叶 s⁻¹)、气孔导度gs、水势、根长密度(cm cm⁻³土)及茎节糖分浓度;群体层登记叶面积指数LAI(m²叶 m⁻²地)、截光比例fIPAR、干物质(t DM ha⁻¹)、蔗产量(t fresh cane ha⁻¹)和糖产量。 必须同时保存分母、时间窗口与含水量口径,禁止把鲜物质吨数与干物质吨数或溶解固形物与可回收糖混算。
English|At cellular scale record chloroplast volume (μm³), plasmodesmata pit-field area (μm²) and enzyme activities with explicit fresh-mass, protein or area denominators. At organ scale record chlorophyll, nitrogen, net leaf assimilation A (μmol CO₂ m⁻² leaf s⁻¹), stomatal conductance, water potential, root-length density (cm cm⁻³ soil) and internode sugar concentration. At stand scale record leaf-area index LAI (m² leaf m⁻² ground), intercepted PAR fraction, dry biomass (t DM ha⁻¹), cane mass (t fresh cane ha⁻¹) and sugar yield. Every value needs its denominator, time window and moisture basis; fresh and dry mass, Brix and recoverable sugar must not be conflated.
6.2 尺度转换的积分与模型条件 | 6.2 Integration and model assumptions
中文|单叶净同化率A是叶面积与时间标准化的局部通量,冠层净同化必须对叶面积分布、光照、温度、气孔限制和昼夜变化积分,并减去不能忽略的呼吸。 可用概念式A_canopy(t)=∫A_leaf(z,t)·dLAI(z)表示结构,但这不是无需校准的甘蔗实测公式。 生物量增量还要扣除呼吸与损耗,再乘以器官分配比例;蔗糖产量还需考虑糖浓度、回收率及杂质。 个体叶片或显微数据缺少这些中介变量,不能直接推算“每公顷增产百分比”。
English|Leaf net assimilation A is a localized flux normalized by leaf area and time. Canopy assimilation requires integration over leaf-area distribution, light, temperature, stomatal limits and diurnal dynamics, with appropriate respiratory accounting. The conceptual relation A_canopy(t) = ∫ A_leaf(z,t) dLAI(z) explains the dimensional bridge, not an uncalibrated sugarcane yield equation. Biomass gain also depends on respiration, losses and allocation; harvested sugar further depends on sucrose concentration, recovery and impurities. Microscopic or individual-leaf measurements without these intermediate variables cannot justify a claimed percentage yield increase per hectare.
6.3 采样设计和伪重复防护 | 6.3 Sampling design and protection against pseudoreplication
中文|每个观测须明确层级:研究地点→区组→小区→植株/分蘖→叶位/节位→组织片→视野→细胞器。 对处理效应的推断,原则上以真正随机分配处理的小区或独立容器为试验单位;同一小区的多叶片是嵌套重复。 RNA-Seq需记录独立植株、技术重复和测序文库;显微数据需同时报告植株数与细胞器数。 拟合混合模型时将地点、区组和植株作为适当的随机或层级项,避免将大量像素当作样本量。
English|Every record needs a hierarchy: site → block → plot → plant/tiller → leaf or internode rank → tissue section → field of view → organelle. Treatment inference generally rests on independently randomized plots or pots. Multiple leaves from one plot are nested subsamples. RNA-Seq requires the number of plants, technical replicates and libraries; microscopy requires both plants and organelles. Hierarchical or mixed models can account for site, block and plant as appropriate. Treating millions of pixels or reads as independent replicates is invalid.
6.4 主张分级和反证保存 | 6.4 Claim grading and preservation of contradictory results
中文|本章将A级用于原始全文直接支持、材料与方法已核清的狭义结论;B级用于摘要或部分原文支持且关键重复信息不全的结论;C级用于理论综合与待实测机制假说。 分级针对每条主张而非整篇论文。 对于“单叶光合越高→糖产量越高”的推论,Irvine结果构成限制而非应剔除的异常值。 遗失的原始重复、外推系数、品种环境信息统一写为null并注明原因;不以假定系数补齐。
English|Grade A denotes a narrowly formulated claim directly supported by inspected primary full text with essential methods identified; B indicates abstract or partial-text support with important design details missing; C indicates mechanistic synthesis requiring tests. Grades apply to claims, not papers. Irvine’s counterexample to the proposition “higher leaf photosynthesis necessarily gives higher sugar yield” is retained as limiting evidence. Missing replicates, transfer coefficients, and genotype–environment metadata are recorded as null with explicit reasons, never filled by plausible-looking estimates.
表 004-2:尺度—指标—误读风险 / Table 004-2: Scale, variable and invalid inference
Scale | Measured quantity | Proper unit | Cannot infer |
|---|---|---|---|
细胞 / Cell | chloroplast μm³ | organelles nested in 3 plants | not yield per hectare |
叶片 / Leaf | A, μmol CO₂ m⁻² s⁻¹ | leaf position × time | not whole-day canopy flux |
茎 / Internode | SuSy activity ratio | internode rank, assay | not direct sucrose export |
根 / Root | root length, cm | rhizotron × plant | not whole-field water uptake |
群体 / Canopy | LAI, intercepted PAR | replicated field plot | not equivalent to leaf A |
S07 真实图像与机制图解 / Authentic images and mechanism illustrations
7.1 真实田间照片的可证明范围 | 7.1 Scope of evidence from a real field photograph
中文|本章复用Kerry Raymond在澳大利亚昆士兰Alberton拍摄的甘蔗田照片(页面报告日期2022-01-26;CC BY 4.0),可辨认群体高度、叶片重叠及冠层上下层的可见结构。 但照片没有明确品种、植株采样编号、光强仪、种植密度和产量数据;不能用其证明叶面积指数、截光比例或品种耐逆差异。 此次采用已存原件并重新计算SHA-256,未重复下载,也不把复用图算作新增研究。
English|The existing field photograph by Kerry Raymond from Alberton, Queensland (creator-reported date 26 January 2022; CC BY 4.0) shows a visible standing cane crop with overlapping leaves and canopy stratification. It lacks verified cultivar, plant IDs, radiometer readings, spacing and yield measurements; thus it cannot validate LAI, interception or stress tolerance. The already stored original is reused with a fresh SHA-256 check, not redownloaded or counted as a new research study.
7.2 真实显微图的图组与测量局限 | 7.2 Authentic micrographs, grouping and limits
中文|本章复用已在第001章收录并核验的KKU甘蔗叶片显微图组合,图内包含干旱与田间持水处理、不同材料、多面板与20 μm比例尺。 面板标签和图尺应保留原样;本章双语注释不得擅改为C4三维叶绿体显微图,也不能由二维切片推算叶绿体体积。 该图与Lee等2023三维论文是不同研究来源,不应以图版数量增加独立证据计数。
English|The chapter reuses a previously verified multi-panel leaf micrograph from KKU material, contrasting field-capacity and drought conditions with labelled panels and a 20 μm scale bar. Original labels and scale bars are preserved. This two-dimensional tissue image must not be relabelled as a 3-D chloroplast reconstruction or used to calculate chloroplast volume. Its study differs from the 2023 3-D anatomical research; multiple panels do not increase the count of independent experiments.
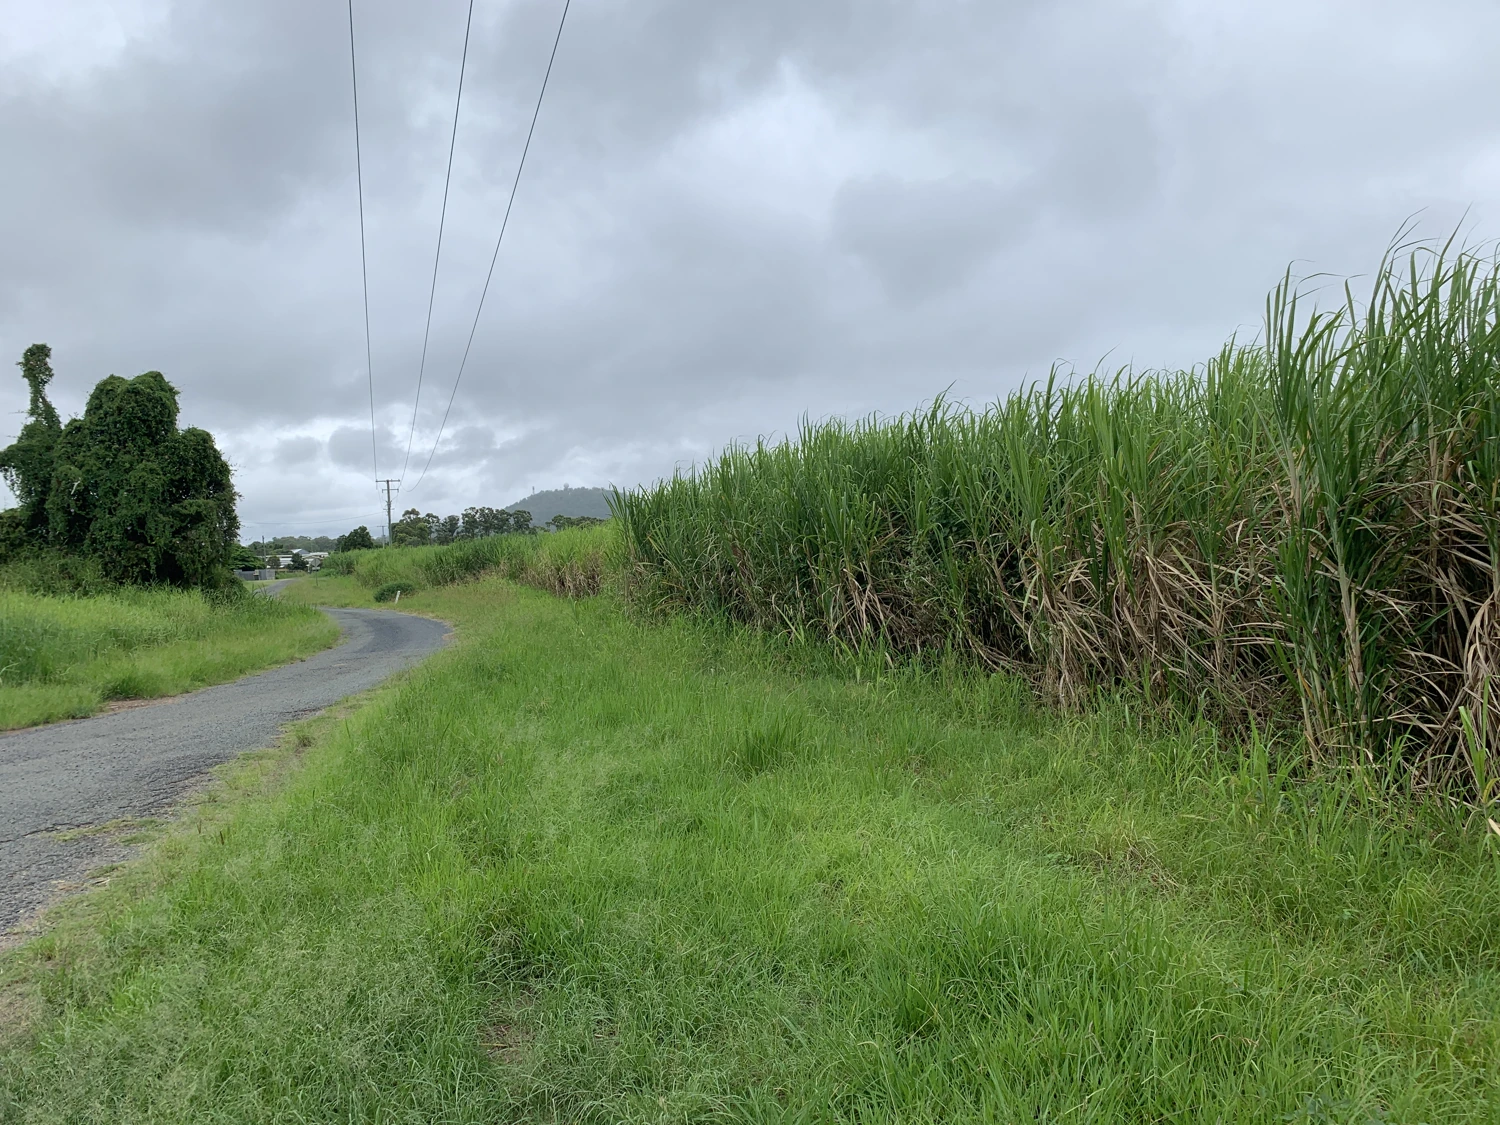
网页预览经过缩放或格式转换,未裁切;原比例尺与标签保留。 / Web preview resized or re-encoded without cropping; original scales and labels retained.
图C004-01。 昆士兰Alberton真实甘蔗田;展示冠层结构,不证明品种、叶面积指数或产量。 作者Kerry Raymond,CC BY 4.0。
Fig. C004-01. Authentic sugarcane field in Alberton, Queensland; illustrates canopy structure, not cultivar, LAI or yield. Kerry Raymond; CC BY 4.0.
Image labels / 图注标签:Field view / 田间实景;cultivar unverified / 品种未核;no scale / 无比例尺。
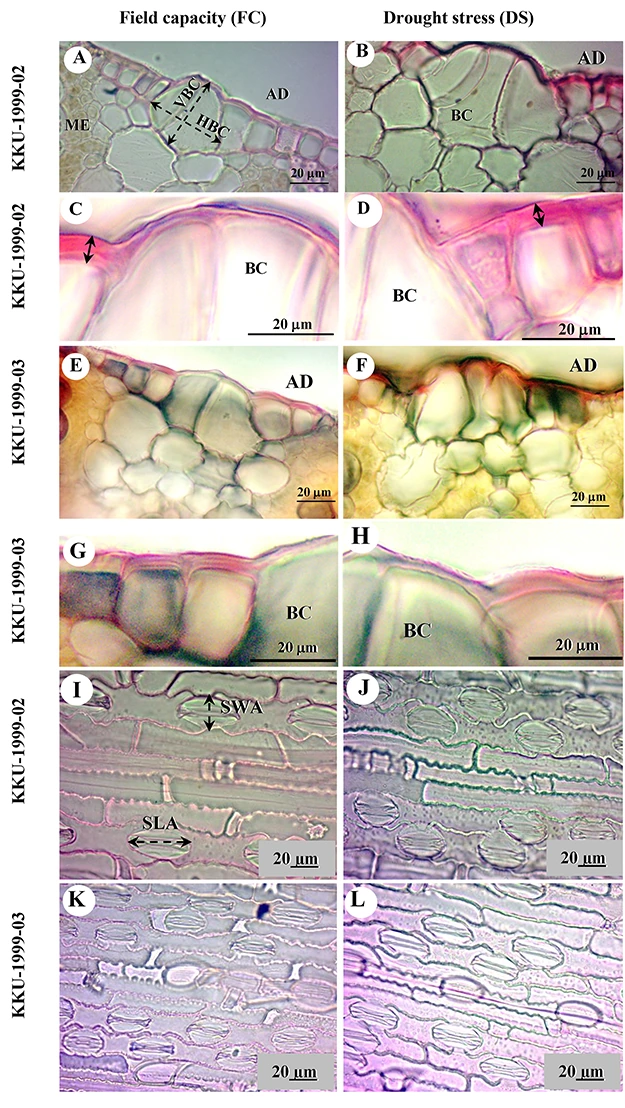
网页预览经过缩放或格式转换,未裁切;原比例尺与标签保留。 / Web preview resized or re-encoded without cropping; original scales and labels retained.
图C004-02。 甘蔗叶组织真实光学显微图(不同基因型×田间持水/干旱处理);各面板比例尺20 μm。 图像仅证明原研究组织形态,不得视为三维叶绿体测量。 原始研究作者Taratima等,CC BY 4.0。
Fig. C004-02. Authentic optical micrographs of sugarcane leaf tissue across genotypes and water treatments; original panel bars = 20 μm. These images are not 3-D chloroplast volumetry. Taratima et al.; CC BY 4.0.
Image labels / 图注标签:FC = field capacity / 田间持水;DS = drought stress / 干旱;20 μm scale bars / 20微米比例尺;original panel labels retained / 原面板标签保留。
S08 适用边界与研究缺口 / Applicability and research gaps
8.1 未被现有证据建立的尺度换算 | 8.1 Scale conversions not established by present evidence
中文|已核读资料可以回答“哪些细胞、组织、叶段或冠层层位存在差异”,但不足以建立全球统一的“叶绿体体积→单叶A→全季节蔗产量”效应链。 更没有证据证明某显微性状跨地区、跨宿根次数具有稳定的经济收益。 缺少的关键环节包括同时测定三维结构、酶活、叶片日积分光合、群体光分布、分配比例、田间鲜蔗与可回收糖,并在多地点多年度进行真正的小区重复。
English|The inspected evidence identifies differences among cell types, tissues, leaf segments and canopy layers, but it does not establish a universal conversion from chloroplast volume to leaf A and finally to season-long cane or sugar yield. Nor does it establish economic benefits across locations or ratoon cycles. Missing links include concurrent 3-D anatomy, enzymology, diurnal leaf exchange, canopy light distribution, allocation, harvested cane and recoverable sugar, with true plot replication across sites and years.
8.2 可重复实施的联合研究方案 | 8.2 A reproducible coordinated research design
中文|建议用至少两个环境、多品种和分层采样设计,在每个独立小区测定冠层PAR剖面与LAI,从相同叶位采集叶片和显微组织,并在相同日期记录土壤水势、叶水势及根长分布;在节间按编号采样测蔗糖与代谢物,最终把逐小区产量和质量检测关联起来。 这里的“两个环境”是拟议方案的最低示范而非来源给定标准;具体重复数要按预期方差和最小可检效应进行事前功效分析。 将盲法图像定量、独立图像校准和缺失数据规则预注册以减少选择性报告。
English|A coordinated design could combine multiple cultivars and at least two environments, sampling a PAR profile and LAI in each independently replicated plot, taking microscopy from matched leaf ranks, and recording soil/leaf water status and roots on aligned dates. Internodes should be ranked for sucrose and metabolites, and plot-level cane yield and quality assessed at harvest. “At least two environments” is an illustrative proposed design, not a literature-derived optimum; formal replication must be determined by prior power analysis. Preregistered image quantification and missing-data rules would reduce selective reporting.
8.3 阶段性结论与审核界限 | 8.3 Provisional conclusions and review boundary
中文|可审阅的阶段性结论是:甘蔗的C4细胞结构具有明确组织分工,同一叶片有生理梯度,节间酶与代谢物随成熟变化,根系对基质的响应因材料不同,冠层光分布与单叶瞬时速率不是相同的量。
English|The defensible interim conclusion is that C4 cellular functions are compartmentalized, leaf blades show developmental gradients, culm enzymes and metabolites change with maturation, roots respond to substrate in genotype-dependent ways, and canopy light distribution is not interchangeable with leaf instantaneous assimilation. Some independent plot counts and raw plant-level observations remain unavailable. This chapter is a research draft with an initial evidence review, not whole-book editorial approval, a yield prescription or authorization to publish on the GAKI website.
双语术语表 / Bilingual terminology
中文 | English |
|---|---|
细胞器 | organelle |
叶肉细胞 | mesophyll cell |
维管束鞘细胞 | bundle-sheath cell |
C4碳浓缩机制 | C4 carbon-concentrating mechanism |
叶绿体容积 | chloroplast volume |
胞间连丝孔域 | plasmodesmata pit field |
磷酸烯醇式丙酮酸羧化酶 | phosphoenolpyruvate carboxylase (PEPC) |
核酮糖-1,5-二磷酸羧化酶/加氧酶 | Rubisco |
叶片气体交换 | leaf gas exchange |
叶面积指数 | leaf area index (LAI) |
冠层净同化 | canopy net assimilation |
冠层光分布 | canopy light distribution |
光合有效辐射 | photosynthetically active radiation (PAR) |
叶片层位 | canopy leaf position |
叶片发育梯度 | leaf developmental gradient |
叶领 | dewlap |
分蘖 | tiller |
节间 | internode |
贮藏薄壁组织 | storage parenchyma |
蔗糖合酶 | sucrose synthase (SuSy) |
源库关系 | source–sink relationship |
韧皮部卸载 | phloem unloading |
根长密度 | root-length density |
根箱 | rhizotron |
宿根蔗 | ratoon crop |
独立实验单位 | independent experimental unit |
生物学重复 | biological replicate |
技术重复 | technical replicate |
嵌套采样 | nested sampling |
伪重复 | pseudoreplication |
标准误 | standard error (SE) |
研究外推边界 | boundary of inference |
原始研究引用 / Original research references
[S01] Lee, Boyd, Boateng & Ort (2023). Exploring 3D leaf anatomical traits for C4 photosynthesis: chloroplast and plasmodesmata pit field size in maize and sugarcane. New Phytologist. DOI: 10.1111/nph.18956. https://nph.onlinelibrary.wiley.com/doi/10.1111/nph.18956. Access scope: FULL_HTML_METHODS_RESULTS. Microscopy fixed/embedded material; shrinkage; not field yield.
[S02] Mattiello et al. (2015). Physiological and transcriptional analyses of developmental stages along sugarcane leaf. BMC Plant Biology. DOI: 10.1186/s12870-015-0694-z. https://link.springer.com/article/10.1186/s12870-015-0694-z. Access scope: FULL_HTML_METHODS_RESULTS. Same-plant paired segments; maize comparison reuses published data.
[S03] James E. Irvine (1975). Relations of Photosynthetic Rates and Leaf and Canopy Characters to Sugarcane Yield. Crop Science. DOI: 10.2135/cropsci1975.0011183X001500050017x. https://acsess.onlinelibrary.wiley.com/doi/abs/10.2135/cropsci1975.0011183X001500050017x. Access scope: PUBLISHER_ABSTRACT. Historic field tests; abstract only; no universal prediction coefficient.
[S04] Marchiori et al. (2010). Plant growth, canopy photosynthesis and light availability in three sugarcane varieties. Sugar Tech. DOI: 10.1007/s12355-010-0031-7. https://connect.eurekamag.com/research/070/570/070570276.php. Access scope: BIBLIOGRAPHIC_ABSTRACT. Secondary abstract index, not full original article.
[S05] Schäfer, Rohwer & Botha (2004). Protein-level expression and localization of sucrose synthase in the sugarcane culm. Physiologia Plantarum. DOI: 10.1111/j.0031-9317.2004.00316.x. https://onlinelibrary.wiley.com/doi/abs/10.1111/j.0031-9317.2004.00316.x. Access scope: PUBLISHER_ABSTRACT. Not direct flux; ratio assay-specific; abstract only.
[S06] Ido et al. (2006). Root growth and distribution of three sugarcane cultivars, in ratoon crop, in two soil types, in rhizotron. Scientia Agraria. DOI: 10.5380/rsa.v7i1.7267. https://revistas.ufpr.br/agraria/article/view/7267/0. Access scope: PUBLISHER_ABSTRACT. Rhizotron confines root space; not direct field uptake.
[S07] Laetsch & Price (1969). Development of the dimorphic chloroplasts of sugar cane. American Journal of Botany. DOI: 10.1002/j.1537-2197.1969.tb07509.x. https://bsapubs.onlinelibrary.wiley.com/doi/epdf/10.1002/j.1537-2197.1969.tb07509.x. Access scope: PUBLISHER_ABSTRACT. Historic microscopy; no quantitative yield tests.
[S08] Authors as published in publisher record (to be confirmed) (2007). Changes in the Sugarcane Metabolome with Stem Development. Are They Related to Sucrose Accumulation?. Plant and Cell Physiology. DOI: 10.1093/pcp/pcm027. https://doi.org/10.1093/pcp/pcm027. Access scope: PUBLISHER_ABSTRACT. Correlations are developmental, not causal enzyme flux.
数据登记 / Associated but non-independent dataset: Mattiello et al. (2015) SRA SRR1979656–SRR1979669, SRR1974519, TSA GCZX00000000 (metadata from original article; no raw sequence files downloaded).
文献不等于试验单位;图版不等于新论文;本章没有提取未经取得的逐株原始观测。 / Papers are not units; image panels are not independent papers; no unavailable raw observations are represented as obtained.